Every discussion of respiration eventually confronts a quiet contradiction. The pathway is introduced as a demolition crew, breaking glucose into carbon dioxide and water to release energy, yet the same intermediates it produces are the raw materials from which cells build fatty acids, amino acids and other essential molecules. A route that both dismantles and constructs cannot honestly be labelled purely catabolic. This lesson examines how fats, glycerol and proteins enter the respiratory pathway at different points, and why that dual traffic justifies calling respiration an amphibolic pathway rather than a catabolic one.
The reasoning rests on a simple but powerful observation. The compounds through which alternative substrates enter the pathway are precisely the compounds that must be withdrawn from it when the organism needs to synthesise those same substrates. Fatty acids are degraded to acetyl CoA before being respired, yet acetyl CoA is also the starting material for fatty acid synthesis. Proteins are dismantled into amino acids whose carbon skeletons feed the Krebs cycle, yet those same skeletons are needed to assemble new proteins. The pathway therefore stands at the crossroads of breakdown and construction, serving both directions of metabolism.
Building on the respiratory balance sheet of the previous lesson, which accounted for the ATP yield of glucose oxidation, this lesson shifts attention from quantity to architecture. It maps the entry points of fats, glycerol and proteins, then reinterprets the entire pathway through the lens of amphibolic function. The terminology and sequence of ideas follow the chapter closely, so that the reasoning arrives where the textbook intends it to arrive. The next lesson will take up the respiratory quotient, where the choice of substrate becomes measurable.
On This Page
Why Glucose Remains the Favoured Respiratory Substrate
Glucose occupies a privileged position in respiration for reasons of convenience as much as chemistry. All carbohydrates are usually first converted into glucose before they are used for respiration, so starch, sucrose and other sugars converge on a single starting point before the pathway proper begins. This convergence simplifies the cell's accounting: one substrate, one set of enzymes, one predictable yield. The respiratory balance sheet of the previous lesson was built entirely on this assumption, counting ATP per molecule of glucose completely oxidised.
Other substrates can also be respired, but they do not enter the respiratory pathway at the first step. This is the crucial qualification. Fats, glycerol and proteins must first be processed into intermediates that the pathway already recognises, and each arrives at a different station along the route. The pathway is therefore less a single entrance than a building with several doors, each admitting a different class of molecule after appropriate preparation. Recognising these doors is the first step towards understanding why the pathway deserves a richer description than "catabolic".
The Convergence of Carbohydrates on Glucose
The conversion of all carbohydrates into glucose before respiration reflects the economy of enzyme reuse. Rather than maintaining separate machinery for every sugar, the cell funnels them into a common intermediate and then applies the standard sequence of glycolysis, the Krebs cycle and the electron transport system. This design means that the energy yield of a polysaccharide can be calculated by first counting its glucose units, a simplification that makes the respiratory balance sheet tractable for students and researchers alike.
This convergence also explains why glucose dominates experimental work on respiration. When biochemists measure oxygen consumption or carbon dioxide release, glucose is the reference substrate against which all others are compared. Any deviation from the glucose pattern signals that a different substrate has entered the pathway at a different point, which is exactly the logic that will later underpin the respiratory quotient. For now, the important point is that glucose defines the baseline route, and alternative substrates are understood by where they join it.
Why Alternative Substrates Matter
Living organisms do not always have glucose at their disposal. Germinating seeds mobilise stored fats, dormant tubers draw on proteins, and starving tissues cannibalise their own structural molecules. In each case, respiration must continue using whatever substrate is available, which requires entry points beyond the first step of glycolysis. The flexibility of the pathway is therefore not a biochemical curiosity but a survival necessity, allowing energy metabolism to proceed when the preferred fuel is scarce.
This flexibility carries a deeper implication. If the pathway accepts multiple substrates at multiple points, then its intermediates are shared currency across many metabolic transactions, not merely way-stations on a one-way road to carbon dioxide. That realisation sets up the central argument of the lesson: the same intermediates that admit alternative substrates during breakdown are the ones withdrawn during synthesis. The pathway's doors swing both ways.
The Entry Points of Fats and Glycerol
Fats present a packaging problem for respiration. A triglyceride is too large and too reduced to enter the pathway directly, so it must first be broken down into glycerol and fatty acids. These two products then take separate routes into the respiratory machinery, arriving at different stations and yielding different amounts of energy. The split is chemically logical: glycerol is a three-carbon alcohol that resembles a sugar fragment, while fatty acids are long hydrocarbon chains that resemble nothing in glycolysis at all.
The divergence of these routes illustrates a general principle of metabolic design. A single storage molecule can be dismantled into components that feed different parts of the same pathway, allowing the cell to balance its use of intermediates. Glycerol joins near the middle of glycolysis, while fatty acids are funnelled through acetyl CoA into the Krebs cycle. Neither enters at the first step, confirming that fats are secondary substrates that must be converted before they can be respired.
Fatty Acids and Acetyl CoA
If fatty acids are to be respired, they are first degraded to acetyl CoA and enter the pathway at that point. The degradation proceeds by sequential removal of two-carbon units, each released as acetyl CoA, which then condenses with oxaloacetate to begin the Krebs cycle. Because fatty acids are highly reduced, their complete oxidation yields substantially more ATP per gram than glucose, a fact reflected in the energy density of stored fat and its value as a long-term reserve in seeds and animals.
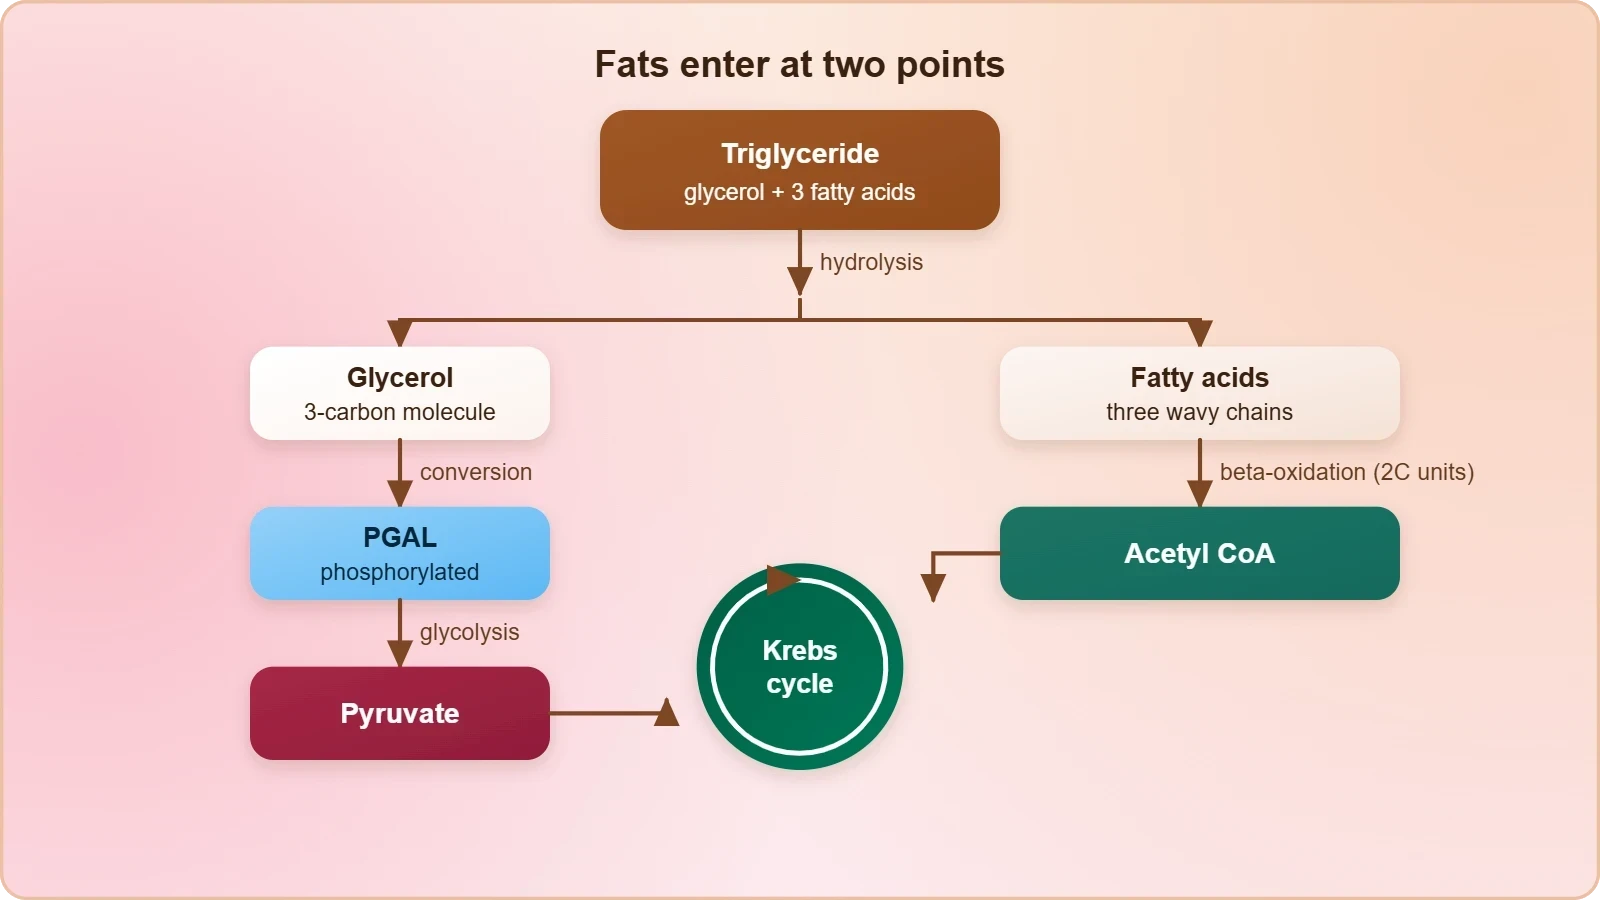
The entry of fatty acids at acetyl CoA rather than at glucose has a consequence worth noting. Acetyl CoA sits at the junction between glycolysis and the Krebs cycle, downstream of the ATP-consuming preparatory phase. Fatty acid oxidation therefore bypasses glycolysis entirely, feeding directly into the cycle that generates reduced coenzymes for the electron transport system. The pathway accommodates this shortcut without difficulty, which is precisely the kind of flexibility the amphibolic concept will later explain.
Glycerol and PGAL
Glycerol follows a shorter route. It enters the pathway after being converted to PGAL, the three-carbon phosphorylated aldehyde also known as glyceraldehyde-3-phosphate, which is a normal intermediate of glycolysis. Once converted, glycerol is indistinguishable from the sugar-derived stream and proceeds through the remainder of glycolysis, pyruvate oxidation and the Krebs cycle like any other carbohydrate fragment. The conversion requires phosphorylation and oxidation, linking glycerol metabolism directly to the mainstream of glucose catabolism.
This entry point is elegant because it requires no new machinery beyond a few familiar enzymes. Glycerol is, in effect, a disguised sugar fragment, and the pathway treats it accordingly. The energy yield is modest compared with fatty acids, but the route is direct. Together, the two halves of a fat molecule demonstrate how a single substrate can be split and routed through different doors of the same pathway, each door positioned where the chemistry fits best.
How Proteins Reach the Respiratory Pathway
Proteins require the most extensive preparation of all the alternative substrates. They are first degraded by proteases into individual amino acids, which cannot be respired as intact molecules. Each amino acid must then be deaminated, meaning its amino group is removed, before its remaining carbon skeleton can be oxidised. Only after this two-stage dismantling does the carbon skeleton become eligible for entry into the respiratory pathway, and the point of entry depends on the structure of the amino acid in question.
This dependence on structure produces a striking diversity of routes. Some amino acids yield carbon skeletons that enter at some stage within the Krebs cycle, slotting in as intermediates such as alpha-ketoglutarate or succinyl CoA. Others are converted to pyruvate, joining the pathway at the junction between glycolysis and the cycle. Still others are degraded to acetyl CoA, entering at the same point as fatty acids. Proteins are therefore not a single substrate but a family of substrates, each with its own door into the pathway.
Deamination and Carbon Skeleton Entry
Deamination is the pivotal step that converts an amino acid from a building block into a fuel. Removing the amino group leaves a carbon skeleton, and it is this skeleton that the respiratory pathway can accept. The nitrogen removed is not wasted; it enters other pathways for disposal or recycling, while the carbon skeleton proceeds towards oxidation. The separation of nitrogen from carbon is what allows protein catabolism to feed into the same energy-yielding machinery used by carbohydrates and fats.
The variety of skeletons explains why proteins can enter at so many points. A carbon skeleton with five carbons may resemble an intermediate of the Krebs cycle; one with three may resemble pyruvate; one with two may resemble acetyl CoA. The pathway recognises these resemblances and absorbs the skeletons accordingly. This adaptability is a further argument against a narrowly catabolic view, since the same intermediates serve as both entry points for degradation and departure points for synthesis.
Pyruvate and Acetyl CoA as Protein Entry Points
When an amino acid is converted to pyruvate, it joins the pathway at the end of glycolysis, where pyruvate would normally be oxidised to acetyl CoA. When it is converted to acetyl CoA, it joins at the entrance to the Krebs cycle. These two entry points are strategically placed at the metabolic crossroads, allowing protein-derived carbon to flow directly into the cycle that generates the reduced coenzymes feeding the electron transport system. The pathway accommodates protein catabolism without any special machinery.
The placement of these entry points also matters for synthesis. Pyruvate and acetyl CoA are not merely fuels; they are precursors for the synthesis of amino acids and fatty acids respectively. An amino acid entering as pyruvate can therefore be reabsorbed into protein synthesis if needed, while acetyl CoA entering from protein can be diverted to fat synthesis. The same junctions serve both directions, which is the essence of the amphibolic argument developed in the next section.
The Case Against a Purely Catabolic View
Since respiration involves breakdown of substrates, the respiratory process has traditionally been considered a catabolic process and the respiratory pathway as a catabolic pathway. The label is understandable: respiration consumes fuel and releases energy, and its most visible outputs are carbon dioxide and water. Yet the chapter asks whether this understanding is correct, and the answer requires looking beyond the direction of net flow to the traffic in both directions along the same route. A road used for deliveries and collections is not accurately described by naming only one direction.
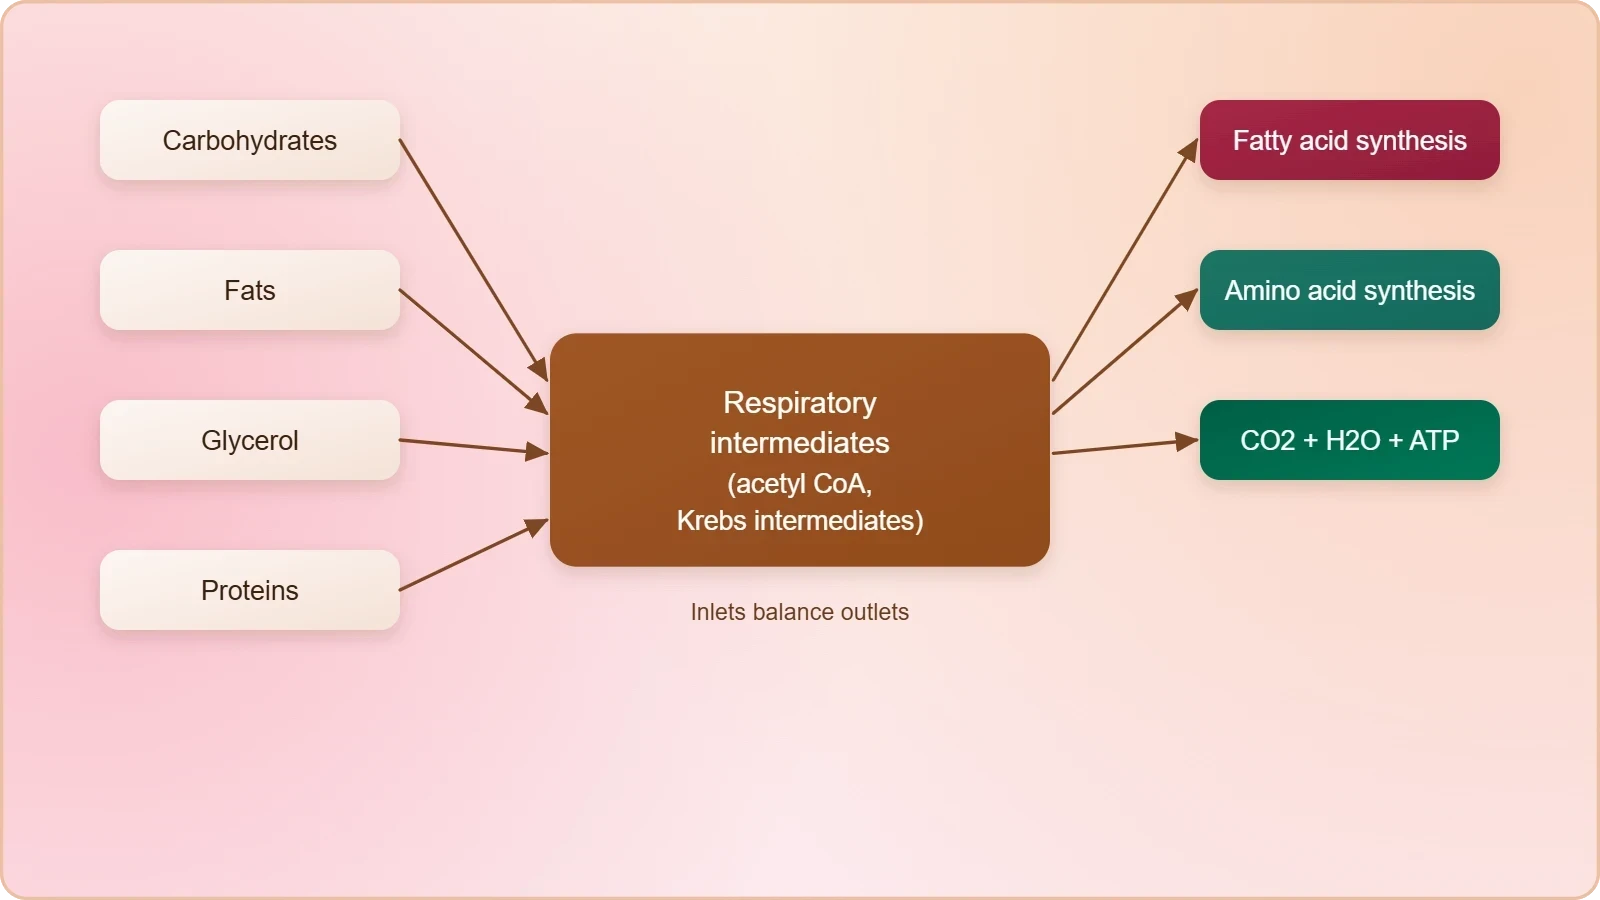
The decisive evidence comes from comparing entry points with withdrawal points. The compounds at which different substrates enter the respiratory pathway are the very compounds that would be withdrawn from it for the synthesis of those substrates. Fatty acids are broken down to acetyl CoA before entering the pathway when used as a substrate, but when the organism needs to synthesise fatty acids, acetyl CoA is withdrawn from the respiratory pathway for that purpose. The pathway therefore comes into the picture both during breakdown and synthesis of fatty acids.
Withdrawal of Intermediates for Synthesis
The withdrawal of intermediates is not an occasional exception but a continuous requirement of biosynthesis. Acetyl CoA leaves the pathway to become the starting unit of fatty acid chains. Krebs cycle intermediates leave to provide carbon skeletons for amino acid synthesis. Even pyruvate can be diverted towards the assembly of new molecules. Every one of these withdrawals must eventually be replenished, or the cycle would stall, which is why cells maintain anaplerotic reactions that top up intermediate pools.
This two-way traffic means that the respiratory pathway cannot be understood as a simple conveyor belt carrying glucose towards carbon dioxide. It is better pictured as a reservoir with many inlets and outlets, where the water level is maintained by balancing inflow against withdrawal. The same molecule may be oxidised for energy today and incorporated into a fatty acid tomorrow, depending on the organism's needs. The pathway's identity is defined by this dual role, not by the direction of its dominant flux.
Protein Synthesis and Respiratory Intermediates
During the breakdown and synthesis of protein too, respiratory intermediates form the link. When proteins are catabolised, their amino acid skeletons enter the pathway at various points; when proteins are anabolised, those same skeletons are drawn from the pathway to build new amino acids. The Krebs cycle intermediates alpha-ketoglutarate, succinyl CoA, fumarate and oxaloacetate are all precursors of amino acid families, making the cycle a hub for both energy release and biosynthetic supply.
This shared use of intermediates is the strongest single argument for the amphibolic label. A pathway that supplies the carbon skeletons for protein synthesis while simultaneously oxidising protein-derived skeletons for energy is performing two opposite functions through one set of reactions. Calling it catabolic captures only half the story. The chapter's conclusion follows directly: because the respiratory pathway is involved in both anabolism and catabolism, it is better considered amphibolic.
Defining the Amphibolic Pathway
Breaking down processes within the living organism are called catabolism, and synthesis is called anabolism. Because the respiratory pathway is involved in both anabolism and catabolism, it is better considered an amphibolic pathway rather than a catabolic one. The term amphibolic captures the dual allegiance directly: the pathway belongs to both halves of metabolism, serving as the shared stage on which breakdown and construction meet. This definition is the conceptual heart of the lesson and the destination towards which all the preceding substrate mapping has been travelling.
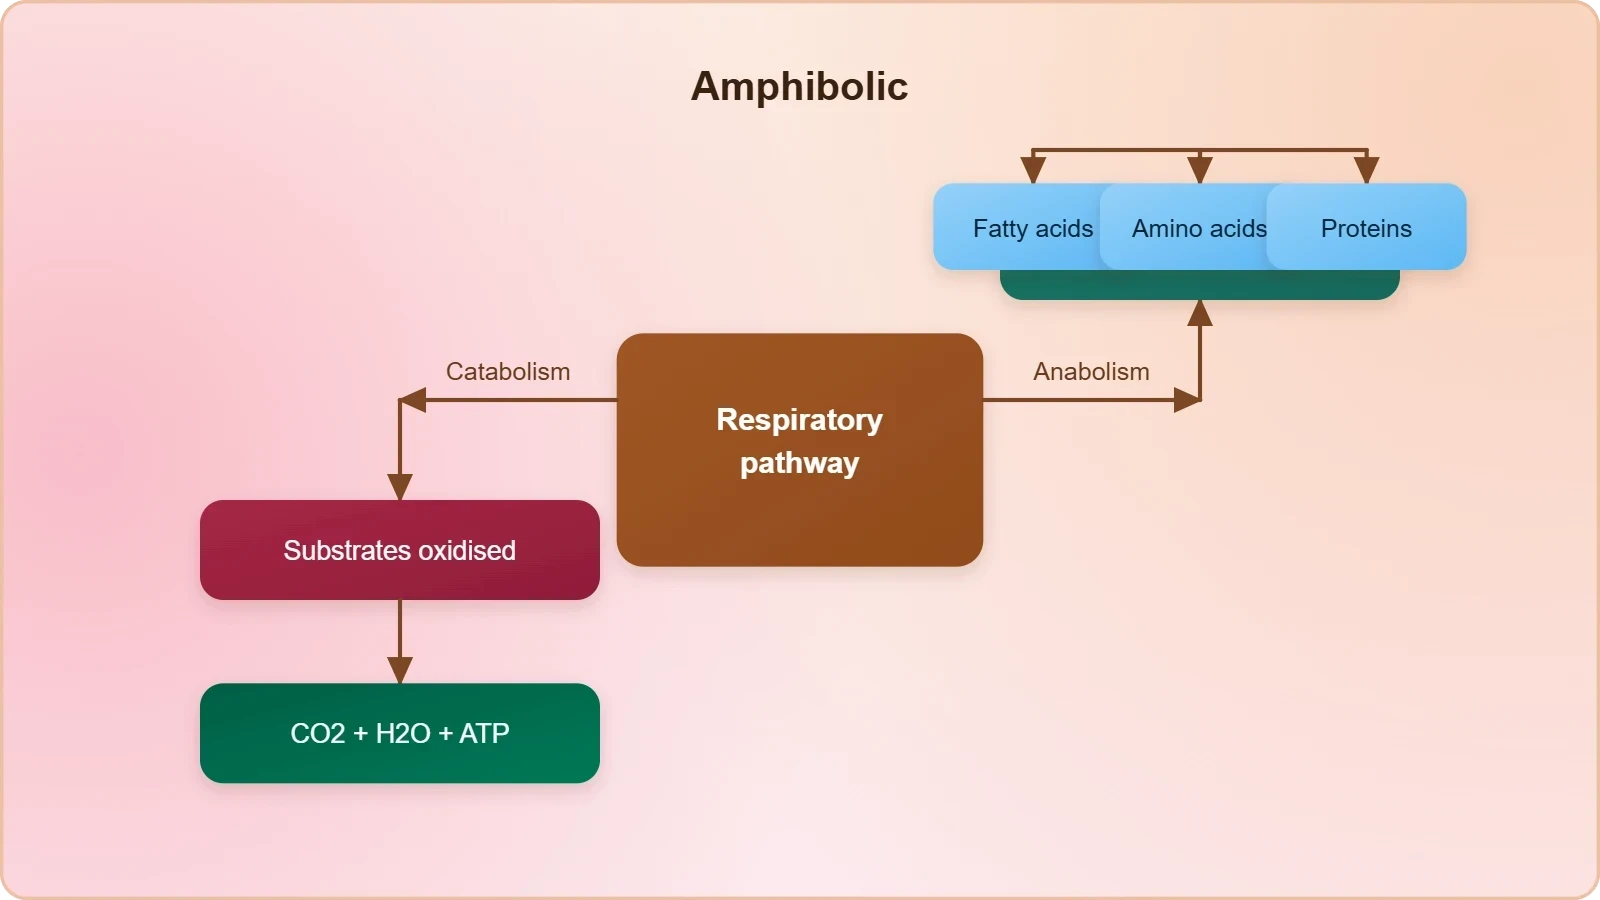
The definition also reframes how the pathway should be studied. A student who sees respiration only as catabolism will be puzzled by the withdrawal of acetyl CoA for fat synthesis or the departure of Krebs intermediates for amino acid assembly. A student who sees it as amphibolic will recognise these events as normal traffic rather than exceptions. The pathway's intermediates are a common pool, drawn upon and replenished according to need, and the pool's level is what matters for continued function.
Catabolism and Anabolism in Balance
The balance between catabolism and anabolism is not fixed. During active growth, anabolic withdrawals may dominate, and the cell must replenish intermediates from other sources to keep the cycle running. During starvation, catabolic flux prevails, and the pathway becomes a net source of energy and carbon for essential functions. The amphibolic description accommodates both states without contradiction, because it names the pathway's capacity rather than its momentary direction.
This balance has a quantitative dimension that connects back to the respiratory balance sheet. The ATP yield calculated for glucose oxidation assumes that all carbon flows through to carbon dioxide and water, but in a growing cell some carbon is withdrawn for synthesis, reducing the net energy yield per molecule of glucose. The balance sheet is therefore an idealisation, useful for understanding the pathway's maximum output but not a complete description of a living cell's metabolism.
Why the Term Matters
The term matters because it corrects a misleading simplification. Describing respiration as purely catabolic encourages the assumption that its intermediates exist only to be oxidised, when in fact they are the raw materials of biosynthesis. The amphibolic label restores the pathway to its proper place at the centre of metabolism, where energy release and molecular construction are two aspects of a single integrated system. It is a small terminological change with substantial explanatory power.
The term also prepares the ground for the next lesson. The respiratory quotient measures the ratio of carbon dioxide released to oxygen consumed, and its value depends on which substrate is being respired. An amphibolic pathway that accepts fats, proteins and carbohydrates at different points will produce different quotients for each, and the interpretation of those quotients requires the substrate map developed here. The amphibolic concept is thus both a conclusion and a bridge.
Working Through the Substrate Routes
Applying the amphibolic concept requires practice in tracing substrates from their storage forms to their entry points. A worked example makes the logic concrete. Consider a triglyceride molecule destined for respiration. It is first broken down into glycerol and fatty acids. The glycerol is converted to PGAL and enters glycolysis; the fatty acids are degraded to acetyl CoA and enter the Krebs cycle. Two products, two doors, one pathway. The same molecule illustrates both the diversity of entry points and the unity of the route they feed.
Now consider the reverse direction. Suppose the organism needs to store fat. Acetyl CoA is withdrawn from the respiratory pathway and used to build fatty acid chains, while glycerol is generated from a glycolytic intermediate. The pathway that yesterday dismantled a fat is today assembling one, using the same intermediates in the opposite direction. This reversibility is the practical meaning of amphibolic, and tracing it through a concrete example makes the abstract term tangible.
Tracing a Fat Molecule Through the Pathway
The fatty acid route begins with degradation to acetyl CoA, a process that releases reduced coenzymes and feeds the Krebs cycle. Each acetyl CoA condenses with oxaloacetate, and the cycle oxidises the two-carbon unit to carbon dioxide while regenerating oxaloacetate. The reduced coenzymes pass electrons to the electron transport system, and oxidative phosphorylation converts the resulting proton gradient into ATP. The energy yield is substantial because fatty acids are highly reduced, packing more electrons per carbon than carbohydrates.
The glycerol route is shorter and less energy-rich. Conversion to PGAL places glycerol in the middle of glycolysis, after the ATP-consuming preparatory phase, so its net yield is slightly higher per carbon than glucose's. From PGAL onwards, the route is identical to the standard glycolytic sequence, proceeding through pyruvate to acetyl CoA and into the Krebs cycle. The two halves of the fat molecule thus converge on acetyl CoA, one directly and one through glycolysis, before completing their oxidation together.
Tracing an Amino Acid Through the Pathway
An amino acid begins its respiratory life as part of a protein. Proteases degrade the protein into individual amino acids, and deamination removes the amino group from each. The remaining carbon skeleton then enters the pathway at a point determined by its structure: within the Krebs cycle, or as pyruvate, or as acetyl CoA. From that entry point, the skeleton is oxidised like any other fuel, yielding reduced coenzymes and eventually ATP through the electron transport system and oxidative phosphorylation.
The same skeleton can also travel in the opposite direction. If the organism needs to synthesise a protein, carbon skeletons are withdrawn from the Krebs cycle and other intermediates and aminated to form amino acids, which are then linked into polypeptide chains. The respiratory pathway thus supplies the raw material for protein synthesis while also disposing of protein breakdown products. This dual traffic, repeated for fats and proteins alike, is the empirical foundation of the amphibolic conclusion.
Going Further
Two background definitions help consolidate the lesson without altering its content. Deamination is the removal of an amino group from an amino acid, leaving a carbon skeleton that the respiratory pathway can accept. Catabolism is the breakdown of molecules, and anabolism is their synthesis. These definitions are standard in biochemistry and simply give precise names to the processes the chapter describes, allowing the amphibolic argument to be stated in formal metabolic language.
Beyond these definitions, it is worth noting that the amphibolic character of respiration is a general feature of central metabolism, not a peculiarity of plants. The same intermediates serve biosynthetic and oxidative roles across organisms, which is why the concept appears throughout biochemistry. The chapter's contribution is to state the idea clearly in the context of plant respiration, using the entry points of fats, glycerol and proteins as evidence. The next lesson turns to the respiratory quotient, where substrate choice becomes measurable.
Also Read
- No links available.
From our network :
- EV 2.0: The Solid-State Battery Breakthrough and Global Factory ExpansionDiscover the impact of the Solid-State Battery Breakthrough on the EV market. Learn about CATL and BYD stock growth, global factory expansion in Europe, and the future of EV 2.0 technology.
- 98% of Global MBA Programs Now Prefer GRE Over GMAT Focus EditionExplore why 98% of global MBA programs now prefer the GRE over GMAT Focus. Learn about the shorter GRE format, verbal logic importance, and strategic versatility for students.
- Analyzing Trump Deportation Numbers Insights Into The 2026 Immigration Crackdown
- Vite 6/7 'Cold Start' Regression in Massive Module GraphsIn-depth analysis of Vite 6/7 cold start regressions in massive module graphs. Learn about barrel file issues, pre-bundling optimizations, and how to improve Vite dev server performance.
- 10 Physics Numerical Problems with Solutions for IIT JEEPrepare for IIT JEE with 10 physics numerical problems, complete with detailed solutions and conceptual explanations. Ideal for mastering kinematics, thermodynamics, electromagnetism, and optics.
- Mastering DB2 12.1 Instance Design: A Technical Deep Dive into Modern Database ArchitectureComprehensive guide to DB2 12.1 Instance Design. Explore architectural components, HADR setup, buffer pool tuning, and security policies for IBM DB2 12.1. Includes 10 functional SQL and Shell samples.
- Trump Political Strategy How Geopolitical Stunts Serve As Media Diversions
- AI-Powered 'Precision Diagnostic' Replaces Standard GRE Score ReportsDiscover the new GRE Precision Diagnostic. Learn how AI-powered behavioral analytics and time-to-solve tracking are replacing standard GRE score reports to empower students.
- Mastering DB2 LUW v12 Tables: A Comprehensive Technical GuideComprehensive guide on DB2 LUW v12 tables. Explore CREATE TABLE syntax, BLU Acceleration, range partitioning, data types, and security features for IBM DB2 LUW v12.
RESOURCES
- Amphibolic Pathway - BYJU'Sbyjus.comRespiration is the breakdown of the complex compounds into simple ones to produce energy molecule, ATP. Hence the process is called catabolic process and…
- respiration in plants chapter 12 - NCERTncert.nic.inthe reaction is very vigorous in case of aerobic respiration. 12.6 AMPHIBOLIC PATHWAY. Glucose is the favoured substrate for respiration. All carbohydrates ...
- Amphibolic - Wikipediaen.wikipedia.orgAll the reactions associated with synthesis of biomolecule converge into the following pathway, viz., glycolysis, the Krebs cycle and the electron transport ...
- Amphibolic Pathway and Respiratory Quotient - Khan Academykhanacademy.orgThis exercise is about how and where different molecules enter the respiratory pathway, how respiration is an amphibolic pathway and the respiratory ...
- Amphibolic Pathway: Definition, Examples, Regulation, Importancemicrobenotes.comMar 24, 2026 ... The amphibolic pathway acts as a functional link between anabolism and catabolism, depending upon cellular needs. When cells are in…
- Why is Krebs' cycle (Respiration) an amphibolic pathway? - CK-12ck12.orgTherefore, because the Krebs' cycle involves both the breakdown (catabolism) and synthesis (anabolism) of molecules, it is considered an amphibolic pathway.
- Amphibolic Pathway | CK-12 Foundationflexbooks.ck12.orgNov 1, 2026 ... Proteins are broken down into amino acids, which after deamination enter the respiratory pathway at various points. Cellular respiration is…
- Respiration is amphibolic pathway." Evaluate the statement.brainly.inMar 11, 2020 ... Amphibolic refers to a process or pathway which is both catabolic and anabolic in nature. Explanation. Glucose is the most…
- Amphibolic pathways - Unacademyunacademy.comThe amphibolic process is best understood through Kreb's cycle. A biological process, cellular respiration is. Glucose breaks down and releases energy via an ...
- Why are amphibolic pathways important? - Lifeeasy Biologybiology.lifeeasy.orgcellular-respiration · plant-respiration. 1 answer. The respiratory pathway is an amphibolic pathway. asked in Plant Respiration by Lifeeasy Biology · plant- ...
- Assertion: Respiratory pathway is an amphibolic pathway. Reasontardigrade.inNov 1, 2019 ... AIIMS 2018: Assertion: Respiratory pathway is an amphibolic pathway. Reason: In respiration, there is breakdown of many substances ...
- Assertion : Respiratory pathway is an amphibolic pathway. Reasonallen.inReason : In respiration, there is breakdown of many substances (catabolism) and synthesis of many substances (anabolism) by respiratory intermediates. A. If ...
- Class 11 Biology MCQ – Respiration in Plants – Amphibolic Pathwaysanfoundry.comThis set of Class 11 Biology Chapter 14 Multiple Choice Questions & Answers (MCQs) focuses on “Respiration in Plants – Amphibolic Pathway”.
- Amphibolic Pathway - GeeksforGeeksgeeksforgeeks.orgJun 23, 2026 ... Respiration is considered an amphibolic pathway because it performs both catabolic and anabolic functions. 1. Catabolic Role of Respiration.
- Assertion: Respiratory pathway is an amphibolic pathway. Reasonvedantu.com... the respiratory pathway. Similarly, proteins are also converted to amino acids which enter respiration after deamination. In the anabolic path- Respiration ...