The tricarboxylic acid cycle occupies the central position in aerobic respiration, and understanding it is essential for anyone who wishes to see how the energy locked inside a glucose molecule is finally released. Once pyruvate has been carried from the cytoplasm into the mitochondrial matrix and converted into acetyl coenzyme A, the stage is set for a remarkable sequence of eight enzyme-catalysed reactions that strip hydrogen atoms from the substrate, release carbon dioxide, and conserve the liberated energy in the form of reduced coenzymes. This lesson follows that cycle step by step, from the condensation of the acetyl group with oxaloacetic acid to the regeneration of the starting material, so that the logic of the pathway becomes clear rather than something to be memorised blindly.
What makes the cycle so instructive is its economy. A single acetyl group, carrying only two carbon atoms, is completely dismantled within one turn, and yet the cell extracts three molecules of NADH, one molecule of FADH2, one molecule of GTP and two molecules of carbon dioxide from that small fragment. The cycle is therefore not merely a disposal route for carbon; it is a precision instrument for harvesting reducing power. Learners who grasp this point will find the later stages of respiration, particularly the electron transport system and oxidative phosphorylation, far easier to follow, because those stages depend entirely on the NADH and FADH2 generated here.
This lesson builds directly on the previous discussion of pyruvate entering the mitochondria and prepares the ground for the next lesson on the electron transport system. It keeps the terminology, the order of ideas and the numerical accounting of the source material intact, while adding a short "Going further" block where well-established background helps the reader place the cycle in a wider context. The aim is a clear, faithful and well-organised account of the tricarboxylic acid cycle that an intermediate learner can study with confidence.
On This Page
- The Tricarboxylic Acid Cycle as the Central Engine of Aerobic Respiration
- The Opening Reactions: Condensation and Isomerisation
- Oxidation of Succinyl-CoA and Regeneration of Oxaloacetic Acid
- Counting the Yield: What One Turn and One Glucose Deliver
- Going Further: Names, Context and the Wider Significance
- Consolidating the Lesson: Structure, Sequence and Significance
The Tricarboxylic Acid Cycle as the Central Engine of Aerobic Respiration
The tricarboxylic acid cycle, more commonly called the Krebs' cycle after the scientist Hans Krebs who first elucidated it, is the cyclic pathway that the acetyl coenzyme A produced from pyruvate enters. Its name derives from the tricarboxylic acids that appear among its intermediates, most notably citric acid, which carries three carboxyl groups. The cycle operates entirely within the matrix of the mitochondrion, the same compartment where pyruvate undergoes oxidative decarboxylation, and it represents the first of the two crucial events of aerobic respiration: the complete oxidation of pyruvate by the stepwise removal of all the hydrogen atoms, leaving three molecules of carbon dioxide.
The second crucial event, the passing on of the electrons removed as part of the hydrogen atoms to molecular oxygen with simultaneous synthesis of ATP, belongs to the inner mitochondrial membrane and will be treated in the next lesson. Keeping these two locations distinct is important. The matrix hosts the decarboxylations and dehydrogenations of the cycle, while the inner membrane hosts the electron transport system. This division of labour explains why the mitochondrion is such an efficient organelle: substrate oxidation and electron transfer are spatially separated yet chemically coupled through the shared pool of NADH and FADH2.
Why a Cycle Rather Than a Straight Chain
The pathway is cyclic because the compound that accepts the acetyl group, oxaloacetic acid, is regenerated at the end of each turn. This design has a profound consequence: a small catalytic quantity of oxaloacetic acid can process an unlimited number of acetyl groups, provided it is continually replenished. The continued oxidation of acetyl coenzyme A via the tricarboxylic acid cycle therefore requires the continued replenishment of oxaloacetic acid, the first member of the cycle. Without that replenishment, the cycle would stall even if acetyl coenzyme A were abundant.
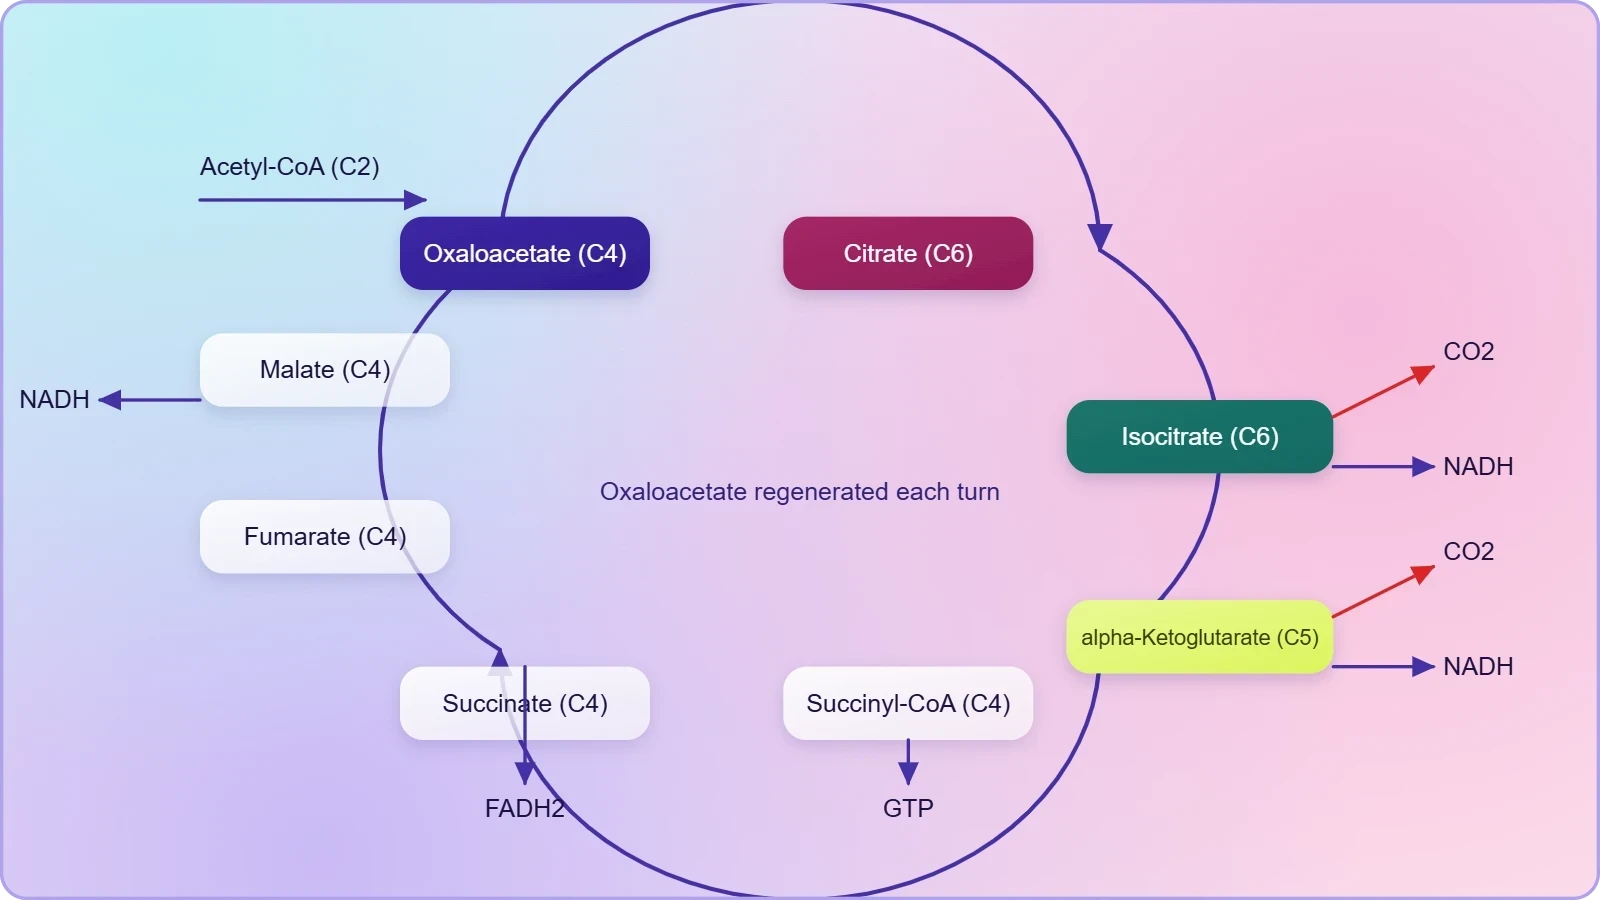
Equally, the cycle requires the regeneration of NAD+ and FAD+ from NADH and FADH2 respectively. If the reduced coenzymes accumulated without being reoxidised, the dehydrogenation steps would have no acceptor and the cycle would halt. This is precisely why oxygen matters: by accepting electrons at the end of the electron transport system, oxygen indirectly keeps NAD+ and FAD+ available, allowing the cycle to continue turning. The cycle and the electron transport system are thus mutually dependent, a point worth holding in mind throughout this lesson.
The Entry Point: Acetyl Coenzyme A
Before the cycle proper begins, pyruvate formed by the glycolytic catabolism of carbohydrates in the cytosol enters the mitochondrial matrix and undergoes oxidative decarboxylation by a complex set of reactions catalysed by pyruvic dehydrogenase. These reactions require the participation of several coenzymes, including NAD+ and coenzyme A. The overall transformation may be written as follows, with the enzyme acting upon pyruvic acid in the presence of coenzyme A, NAD+ and magnesium ions:
During this process, two molecules of NADH are produced from the metabolism of two molecules of pyruvic acid, since one glucose molecule yields two pyruvic acid molecules during glycolysis. The acetyl coenzyme A so formed then enters the cyclic pathway. It is worth noting that the carbon dioxide released at this step is the first of the three molecules that will ultimately leave each pyruvate, and that the acetyl group itself carries only two carbon atoms into the cycle, the third having already departed as carbon dioxide.
The Opening Reactions: Condensation and Isomerisation
The tricarboxylic acid cycle starts with the condensation of the acetyl group with oxaloacetic acid and water to yield citric acid. The reaction is catalysed by the enzyme citrate synthase, and a molecule of coenzyme A is released in the process. This is the defining moment of the cycle: the two-carbon acetyl unit is joined to the four-carbon oxaloacetic acid, producing a six-carbon tricarboxylic acid. The release of coenzyme A is significant because it frees the carrier to participate again in the oxidative decarboxylation of further pyruvate molecules, keeping the supply of acetyl coenzyme A flowing.
Citrate is then isomerised to isocitrate. This seemingly modest rearrangement is essential, because it repositions the hydroxyl group so that the subsequent oxidative decarboxylations can proceed. The isomerisation is a reminder that the cycle is not a simple sequence of degradations but a carefully choreographed set of transformations in which the geometry of the substrate is adjusted at each stage to permit the next enzyme to act. Learners should appreciate that the six-carbon stage is short-lived and serves mainly as a scaffold from which two carbon atoms will soon be removed.
Two Successive Decarboxylations
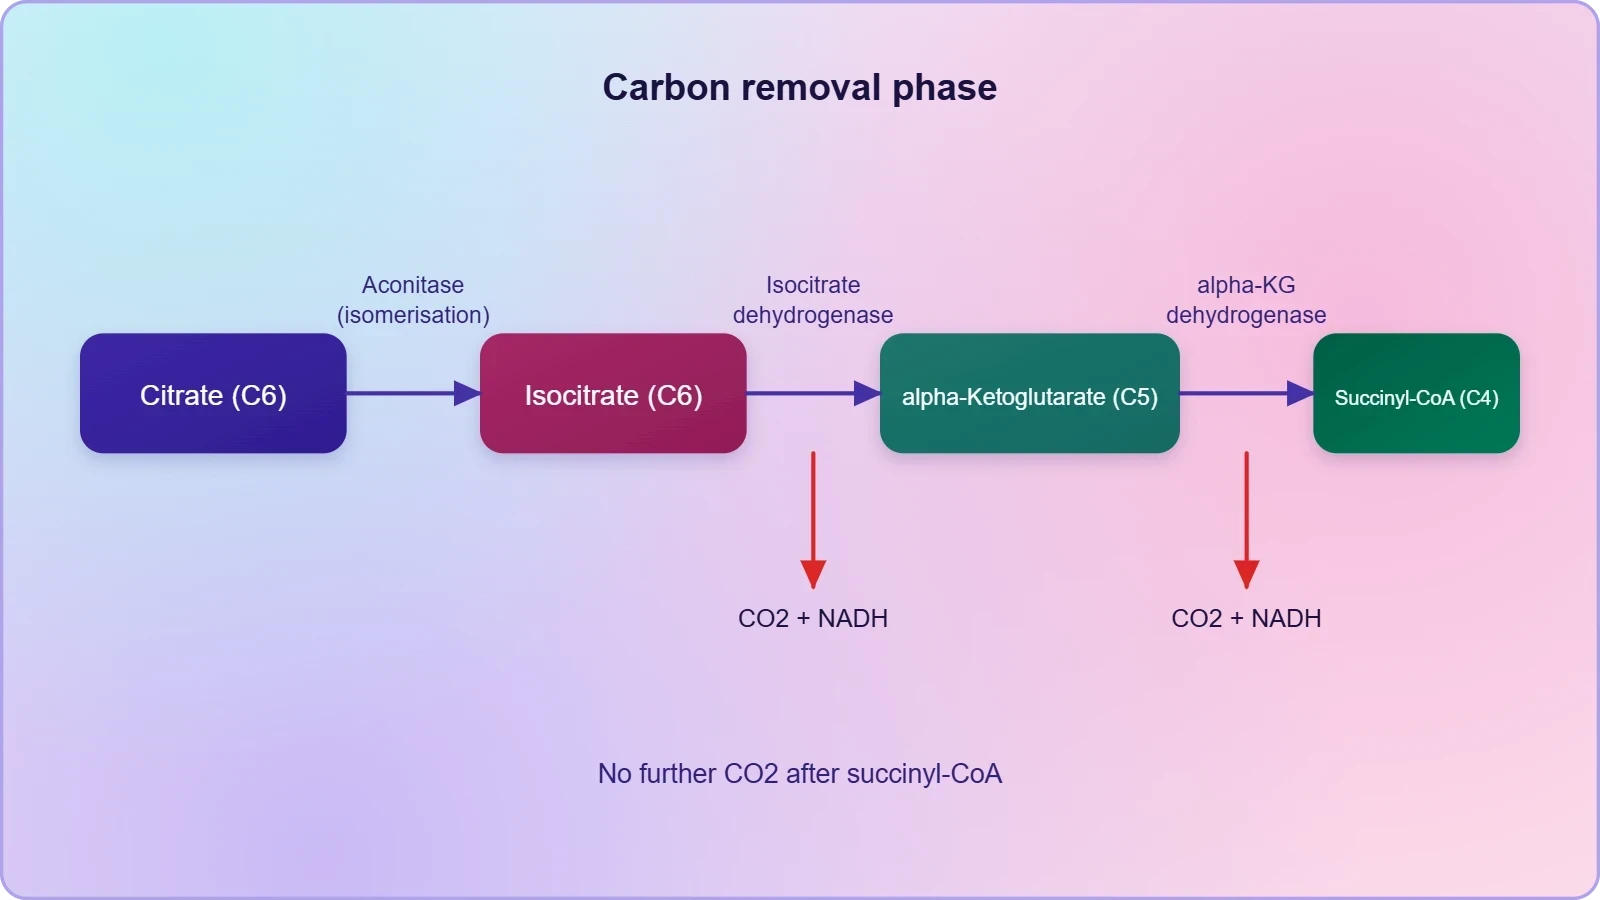
The isomerisation of citrate to isocitrate is followed by two successive steps of decarboxylation, leading to the formation of α-ketoglutaric acid and then succinyl-CoA. In these steps the six-carbon skeleton is progressively trimmed: the first decarboxylation removes one carbon atom to leave the five-carbon α-ketoglutaric acid, and the second removes another to leave the four-carbon succinyl-CoA. Each decarboxylation is accompanied by a dehydrogenation, so that NAD+ is reduced to NADH + H+ at both stages. The carbon dioxide released here, together with that released during the oxidative decarboxylation of pyruvate, accounts for the three molecules of carbon dioxide produced per pyruvate.
The formation of succinyl-CoA marks the completion of the carbon-removal phase of the cycle. From this point onward, no further carbon dioxide is released; the remaining steps are concerned with oxidising the four-carbon unit back to oxaloacetic acid and conserving the energy released in the process. This division of the cycle into a decarboxylating phase and an oxidising phase is a useful way to organise one's understanding, and it mirrors the broader logic of aerobic respiration, in which carbon is first stripped away and the resulting reducing power is then converted into ATP.
Energy Conservation at the Succinyl-CoA Step
In the remaining steps of the citric acid cycle, succinyl-CoA is oxidised to oxaloacetic acid, allowing the cycle to continue. During the conversion of succinyl-CoA to succinic acid, a molecule of GTP is synthesised. This is a substrate level phosphorylation. In a coupled reaction, GTP is converted to GDP with the simultaneous synthesis of ATP from ADP. The term substrate level phosphorylation is precise: the phosphate group is transferred directly from a substrate molecule to a nucleotide, without the involvement of the electron transport system or a proton gradient.
This step is the only point in the cycle where a nucleotide triphosphate is formed directly. All the other energy conserved during the cycle is captured in the reduced coenzymes NADH + H+ and FADH2, which will later be oxidised through the electron transport system. The distinction matters because it explains why the cycle on its own yields only a modest amount of ATP directly, while its true energetic contribution is realised only when the reduced coenzymes are processed by the inner mitochondrial membrane.
Oxidation of Succinyl-CoA and Regeneration of Oxaloacetic Acid
After the decarboxylation phase, the cycle turns to the task of regenerating oxaloacetic acid from the four-carbon intermediate succinyl-CoA. Succinyl-CoA is converted to succinic acid, and in the process a molecule of GTP is synthesised by substrate level phosphorylation. Succinic acid is then oxidised to fumaric acid, with FAD+ acting as the hydrogen acceptor and being reduced to FADH2. This is the single point in the cycle where FAD+ rather than NAD+ serves as the electron acceptor, a detail that learners should note carefully because it affects the later ATP yield.
Fumaric acid is then hydrated to malic acid, and malic acid is finally oxidised to oxaloacetic acid, with NAD+ reduced to NADH + H+. With the regeneration of oxaloacetic acid, the cycle is complete and ready to accept another acetyl group. The continued oxidation of acetyl coenzyme A via the tricarboxylic acid cycle requires the continued replenishment of oxaloacetic acid, the first member of the cycle, and it also requires the regeneration of NAD+ and FAD+ from NADH and FADH2 respectively. These two requirements are the operational constraints that govern the cycle's activity.
Three Points of NAD+ Reduction and One of FAD+ Reduction
There are three points in the cycle where NAD+ is reduced to NADH + H+ and one point where FAD+ is reduced to FADH2. The three NAD+-linked steps occur at the oxidation of isocitrate to α-ketoglutaric acid, at the oxidation of α-ketoglutaric acid to succinyl-CoA, and at the oxidation of malic acid to oxaloacetic acid. The single FAD+-linked step occurs at the oxidation of succinic acid to fumaric acid. This distribution is a fixed feature of the cycle and is central to the respiratory balance sheet that will be examined later in the course.
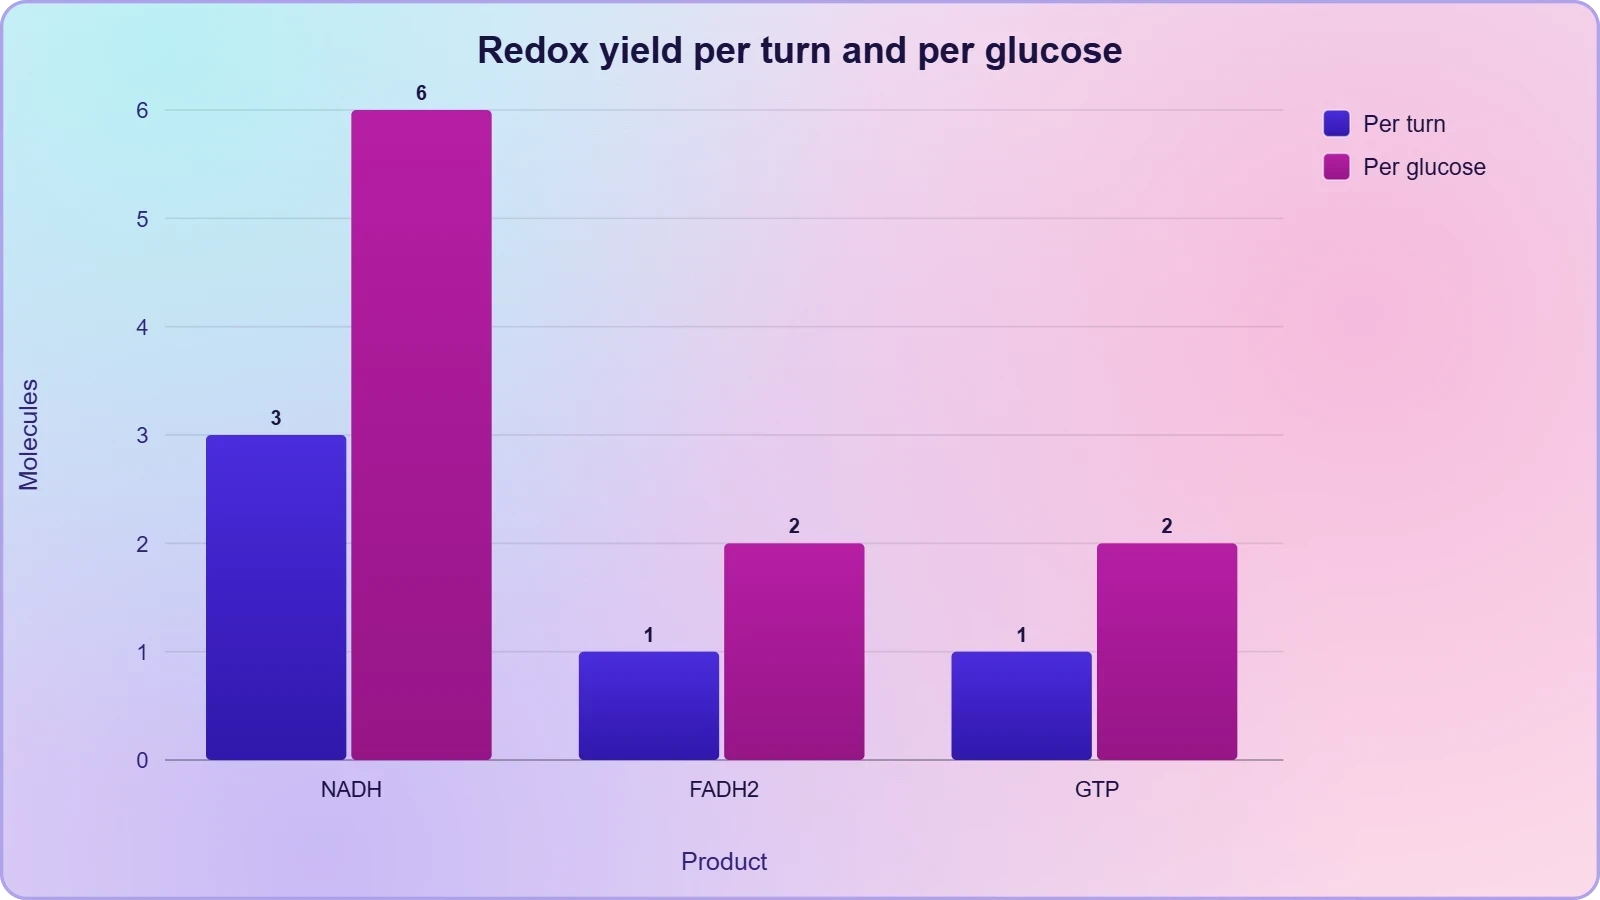
Because each turn of the cycle processes one acetyl group, and each glucose molecule yields two acetyl groups, the cycle turns twice per glucose molecule. The reduced coenzymes produced in a single turn are therefore doubled when accounting for a whole glucose molecule. This doubling is the source of the eight molecules of NADH + H+ and two molecules of FADH2 that the cycle contributes per glucose, figures that will be combined with those from glycolysis and the link reaction in the respiratory balance sheet.
The Summary Equation for This Phase
The overall transformation accomplished by the cycle can be summarised in a single equation. Pyruvic acid, in the presence of NAD+, FAD, water, ADP and inorganic phosphate, is converted to carbon dioxide, NADH + H+, FADH2 and ATP within the mitochondrial matrix. The equation captures the essential inputs and outputs of the phase and serves as a compact reference for revision:
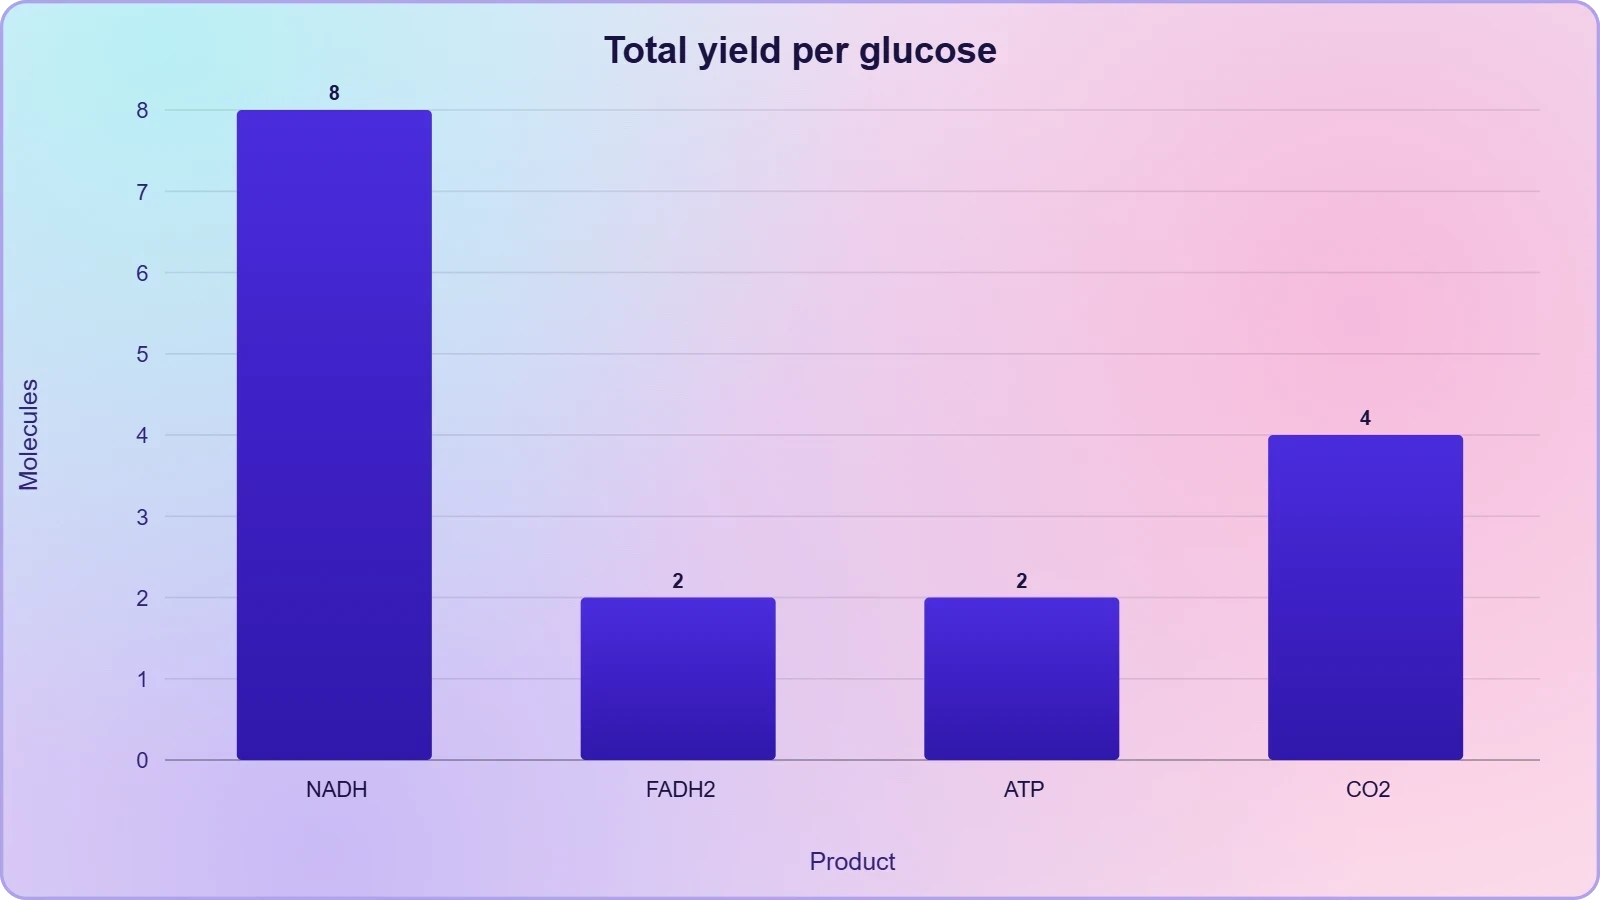
It is important to read this equation in the context of the whole pathway. Glucose has been broken down to release carbon dioxide, and eight molecules of NADH + H+ and two of FADH2 have been synthesised besides just two molecules of ATP in the tricarboxylic acid cycle. Neither oxygen nor the promised large number of ATP molecules has yet appeared. The role of the reduced coenzymes, and the role of oxygen in reoxidising them, is the subject of the next lesson.
Counting the Yield: What One Turn and One Glucose Deliver
Keeping a clear tally of the products is one of the most practical skills a learner can develop for this topic. In a single turn of the cycle, one acetyl group yields two molecules of carbon dioxide, three molecules of NADH + H+, one molecule of FADH2 and one molecule of GTP, which is converted to ATP in a coupled reaction. Since one glucose molecule produces two pyruvic acid molecules, and each pyruvate yields one acetyl coenzyme A, the cycle turns twice per glucose. Doubling the single-turn figures gives the cycle's total contribution per glucose molecule.
That total is four molecules of carbon dioxide, six molecules of NADH + H+, two molecules of FADH2 and two molecules of ATP. When the NADH produced during the oxidative decarboxylation of the two pyruvates is added, the figure rises to eight molecules of NADH + H+, which is exactly the number stated in the source material. The two molecules of ATP formed in the cycle are the only ATP generated directly at this stage; everything else is stored in the reduced coenzymes and awaits the electron transport system.
Why the Direct ATP Yield Seems Small
At first sight, two ATP molecules from an entire glucose molecule appear disappointing. The apparent shortfall is resolved once the reduced coenzymes are taken into account. Each NADH + H+ and each FADH2 carries electrons at a high energy level, and when these electrons are passed along the electron transport system to oxygen, a large amount of ATP is synthesised by oxidative phosphorylation. The cycle's real contribution is therefore the reducing power it generates, not the small quantity of ATP it makes directly.
This is why the cycle is described as the central engine of aerobic respiration. It completes the oxidation of the substrate, releasing all the carbon as carbon dioxide, and it funnels the extracted hydrogen into carriers that the inner membrane can process. Without the cycle, glycolysis would leave the cell with a pile of reduced coenzymes and no efficient way to reoxidise them, and the large ATP yield promised by aerobic respiration would never materialise.
Regeneration Requirements and Their Consequences
The cycle can continue only if oxaloacetic acid is replenished and if NAD+ and FAD+ are regenerated from their reduced forms. These requirements link the cycle tightly to the availability of oxygen, because oxygen is the final electron acceptor that allows NADH and FADH2 to be reoxidised. When oxygen is scarce, the reduced coenzymes accumulate, the dehydrogenation steps lose their acceptor, and the cycle slows. This is the biochemical reason why aerobic respiration cannot proceed without oxygen, even though oxygen itself does not appear as a reactant in the cycle's own equation.
Understanding this dependency also clarifies the relationship between the cycle and the next lesson. The electron transport system and oxidative phosphorylation exist precisely to reoxidise the NADH + H+ and FADH2 that the cycle produces. The two processes are therefore partners in a continuous loop: the cycle supplies reduced coenzymes, the electron transport system regenerates the oxidised forms, and the cycle can then continue. Recognising this partnership is the key to seeing aerobic respiration as an integrated whole rather than a list of separate reactions.
Going Further: Names, Context and the Wider Significance
The tricarboxylic acid cycle is also called the citric acid cycle or Krebs' cycle. All three names refer to the same pathway, and each highlights a different feature: the tricarboxylic acids that are its intermediates, the citric acid formed at the opening condensation, and the scientist who first elucidated the sequence. Encountering different names in different textbooks can be confusing, so it is worth fixing the equivalence firmly in mind. The abbreviation TCA cycle is also widely used and appears in the source material alongside the full name.
Substrate level phosphorylation is ATP (or GTP) synthesis directly from a substrate during a reaction. The conversion of succinyl-CoA to succinic acid, with the accompanying synthesis of GTP, is the classic example within the cycle. This mechanism contrasts with oxidative phosphorylation, in which ATP is synthesised indirectly, driven by the proton gradient established as electrons pass along the electron transport system. Recognising the distinction helps the learner appreciate why the cycle's direct ATP contribution is modest while its indirect contribution, through the reduced coenzymes, is very large.
Placing the Cycle in the Wider Metabolic Map
Beyond its role in energy release, the cycle is a meeting point for the metabolism of carbohydrates, fats and proteins, since their breakdown products can feed into it at various points. This wider role explains why the cycle is sometimes described as amphibolic, a term introduced later in the course. For the present lesson, the essential point is that the cycle is not an isolated loop but a hub through which many metabolic routes pass, and its intermediates must therefore be replenished from time to time to keep it running.
The cycle also illustrates a general principle of cellular economy: energy is released in small, controlled steps rather than in a single burst. Each decarboxylation and each dehydrogenation releases a modest amount of energy, which is captured in a carrier molecule rather than dissipated as heat. This stepwise strategy is what allows the cell to store energy efficiently and to regulate the rate of respiration in response to its needs, and it is a theme that recurs throughout the study of metabolism.
Preparing for the Electron Transport System
The cycle leaves the cell with a substantial store of reducing power in the form of NADH + H+ and FADH2. The next lesson examines how these carriers are oxidised through the electron transport system, how the electrons are passed on to molecular oxygen to form water, and how the resulting proton gradient drives the synthesis of ATP by oxidative phosphorylation. The figures established here, eight NADH + H+ and two FADH2 per glucose, will be the inputs to that final accounting.
Learners who have followed the cycle carefully will find the next stage easier to grasp, because the logic is continuous: the cycle extracts hydrogen, the carriers transport it, the membrane converts the electrons into a gradient, and the gradient drives ATP synthesis. Each stage depends on the one before it, and the whole sequence is held together by the recycling of NAD+ and FAD+. With this foundation in place, the respiratory balance sheet and the concept of the respiratory quotient become natural extensions rather than isolated facts to be memorised.
Consolidating the Lesson: Structure, Sequence and Significance
The tricarboxylic acid cycle can be held in memory as a sequence of three phases. The first phase is the opening condensation of the acetyl group with oxaloacetic acid and water to yield citric acid, catalysed by citrate synthase, followed by the isomerisation of citrate to isocitrate. The second phase is the pair of successive decarboxylations that produce α-ketoglutaric acid and then succinyl-CoA, releasing two molecules of carbon dioxide and reducing NAD+ at each stage. The third phase is the oxidation of succinyl-CoA back to oxaloacetic acid, during which GTP, FADH2 and a further NADH + H+ are generated.
This three-phase structure is not merely a memory aid; it reflects the chemical logic of the pathway. Carbon is removed first, then the remaining skeleton is oxidised, and finally the starting material is regenerated so that the cycle can begin again. Each phase is catalysed by a distinct set of enzymes, and each contributes a characteristic share of the total yield. Learners who can reproduce this structure from memory, together with the location of the three NAD+-linked steps and the single FAD+-linked step, will have a secure grasp of the cycle.
Common Points of Confusion
Several details are frequently confused. The first is the distinction between the oxidative decarboxylation of pyruvate, which occurs before the cycle and is catalysed by pyruvate dehydrogenase, and the decarboxylations within the cycle itself. The second is the identity of the carbon dioxide-producing steps: two molecules of carbon dioxide are released within the cycle, and the third is released during the formation of acetyl coenzyme A. The third is the single FAD+-linked step at succinic acid, which is easily overlooked because most steps use NAD+.
A fourth point concerns the GTP formed at the succinyl-CoA step. It is synthesised by substrate level phosphorylation and is converted to ATP in a coupled reaction, so the cycle's direct nucleotide yield is one ATP equivalent per turn. A fifth point is the requirement for continual replenishment of oxaloacetic acid and regeneration of NAD+ and FAD+. Keeping these five points clear will prevent most errors in examination answers and will make the respiratory balance sheet much easier to construct when it is reached later in the course.
Looking Ahead to the Balance Sheet
The figures assembled in this lesson feed directly into the respiratory balance sheet, which will combine the yields from glycolysis, the link reaction and the cycle before adding the contribution of oxidative phosphorylation. The cycle's contribution of six NADH + H+, two FADH2 and two ATP per glucose, together with the two NADH from pyruvate oxidation, forms the largest single block of reducing power in the entire pathway. Understanding where each of these molecules comes from is therefore essential preparation for that final accounting.
With the cycle complete, the stage is set for the electron transport system and oxidative phosphorylation, where the energy stored in these carriers is finally converted into the large number of ATP molecules needed for cellular metabolism. The cycle has done its work: the carbon has been released as carbon dioxide, the hydrogen has been captured in carriers, and the cell is ready to cash in that stored reducing power. The next lesson follows exactly that transaction, completing the account of aerobic respiration that began with glycolysis.
Also Read
- No links available.
From our network :
- 98% of Global MBA Programs Now Prefer GRE Over GMAT Focus EditionExplore why 98% of global MBA programs now prefer the GRE over GMAT Focus. Learn about the shorter GRE format, verbal logic importance, and strategic versatility for students.
- Mastering DB2 12.1 Instance Design: A Technical Deep Dive into Modern Database ArchitectureComprehensive guide to DB2 12.1 Instance Design. Explore architectural components, HADR setup, buffer pool tuning, and security policies for IBM DB2 12.1. Includes 10 functional SQL and Shell samples.
- Analyzing Trump Deportation Numbers Insights Into The 2026 Immigration Crackdown
- EV 2.0: The Solid-State Battery Breakthrough and Global Factory ExpansionDiscover the impact of the Solid-State Battery Breakthrough on the EV market. Learn about CATL and BYD stock growth, global factory expansion in Europe, and the future of EV 2.0 technology.
- AI-Powered 'Precision Diagnostic' Replaces Standard GRE Score ReportsDiscover the new GRE Precision Diagnostic. Learn how AI-powered behavioral analytics and time-to-solve tracking are replacing standard GRE score reports to empower students.
- Vite 6/7 'Cold Start' Regression in Massive Module GraphsIn-depth analysis of Vite 6/7 cold start regressions in massive module graphs. Learn about barrel file issues, pre-bundling optimizations, and how to improve Vite dev server performance.
- Mastering DB2 LUW v12 Tables: A Comprehensive Technical GuideComprehensive guide on DB2 LUW v12 tables. Explore CREATE TABLE syntax, BLU Acceleration, range partitioning, data types, and security features for IBM DB2 LUW v12.
- Trump Political Strategy How Geopolitical Stunts Serve As Media Diversions
- 10 Physics Numerical Problems with Solutions for IIT JEEPrepare for IIT JEE with 10 physics numerical problems, complete with detailed solutions and conceptual explanations. Ideal for mastering kinematics, thermodynamics, electromagnetism, and optics.
RESOURCES
- The citric acid cycle | Cellular respiration (article) - Khan Academykhanacademy.orgIn eukaryotes, the citric acid cycle takes place in the matrix of the mitochondria, just like the conversion of pyruvate to acetyl CoA …
- Physiology, Krebs Cycle - StatPearls - NCBI Bookshelfncbi.nlm.nih.govNov 23, 2022 ... The tricarboxylic acid (TCA) cycle, also known as the Krebs or citric acid cycle, is an important cell's metabolic hub…
- Citric acid cycle - Wikipediaen.wikipedia.orgThe citric acid cycle—also known as the Krebs cycle, Szent–Györgyi–Krebs cycle, or TCA cycle (tricarboxylic acid cycle)—is a series of biochemical reactions ...
- Citric Acid Cycle - an overview | ScienceDirect Topicssciencedirect.comThe TCA cycle, also known as the citric acid cycle or Krebs cycle, is defined as a series of biochemical reactions in the mitochondria…
- Evolution and Functional Implications of the Tricarboxylic Acid Cycle ...pmc.ncbi.nlm.nih.govFinally, we performed coexpression analysis using mitochondrial TCA cycle genes revealing close connections among these genes most likely related to the higher ...
- Citric Acid Cycle - an overview | ScienceDirect Topicssciencedirect.comThe TCA cycle, also known as the citric acid cycle, is defined as the central oxidative pathway for the metabolism of carbohydrates, fats, and…
- Global Transcription Analysis of Krebs Tricarboxylic Acid Cycle ...pmc.ncbi.nlm.nih.govThe Krebs tricarboxylic acid (TCA1) cycle is a central pathway of metabolism. Its main catalytic function is to provide reducing equivalents to the respiratory ...
- QuickGO::Term GO:0006099 - Tricarboxylic acid cycleebi.ac.ukDefinition (GO:0006099 GONUTS page). A nearly universal metabolic pathway in which the acetyl group of acetyl coenzyme A is effectively oxidized to two CO2…
- Mitochondrial TCA cycle metabolites control physiology and diseasenature.comJan 3, 2020 ... The TCA cycle, also known as the citric acid cycle or the Krebs cycle, is a series of reactions in…
- Tricarboxylic Acid (TCA) Cycle Intermediates: Regulators of Immune ...pubmed.ncbi.nlm.nih.govJan 19, 2021 ... The tricarboxylic acid cycle (TCA) is a series of chemical reactions used in aerobic organisms to generate energy via the…
- Tricarboxylic Acid Cycle Antibody Sampler Kit #47767cellsignal.comWestern blot analysis of extracts from various cell lines using DLST ... ACO2; Citrate Synthase; DLST; Fumarase; IDH1; IDH2; Krebs; Krebs cycle; MPC1 ...
- Tricarboxylic Acid Cycle Intermediates and Individual Ageingpubmed.ncbi.nlm.nih.govFeb 22, 2024 ... ... explained. This review describes convincingly the ... MeSH terms. Aging / metabolism; Animals; Caenorhabditis elegans; Citric Acid Cycle* ...
- Regulation and function of the mammalian tricarboxylic acid cyclejbc.orgA simplified schematic depicting the reductive TCA cycle or reverse Krebs cycle. Most reactions of this cycle are the same as those of the…
- TCA cycle (aka Krebs or citric acid cycle) (WP78) - Homo sapienswikipathways.orgActivity. last edited · pathway curation. Discuss this pathway. Check for ongoing discussions or start your own. Cited In.