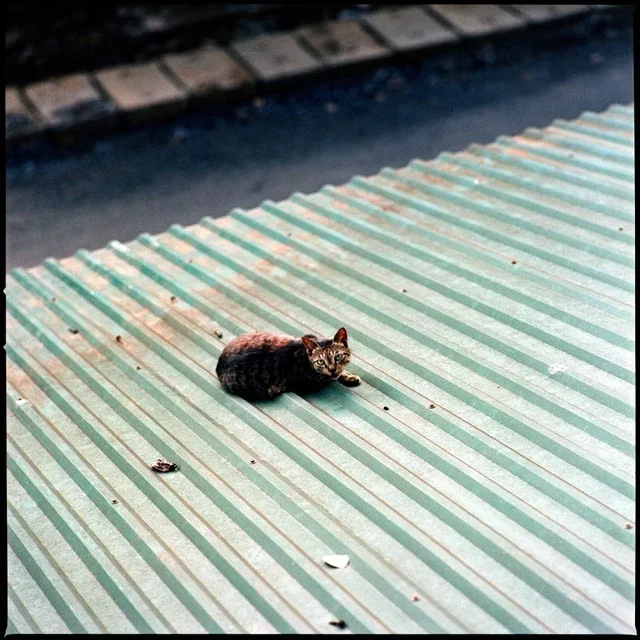
Scholarly inquiry into feline behavioral ecology and chemical communication has recently revealed remarkable dimensions of biochemical signaling within domestic cat populations. Investigators examining biological excretions have identified what can be accurately characterized as an identification-like signature encoded directly within feline urine markers. This sophisticated biomarker functions as a molecular passport, broadcasting complex intraspecific details across territorial boundaries without requiring direct physical confrontation between individual animals.
Feline chemical communication represents an extraordinary evolutionary adaptation that relies heavily on volatile and non-volatile organic compounds deposited strategically within the environment. When researchers analyze the chemical profile of these secretions, they uncover distinct molecular motifs that remain stable across specific temporal windows. These biological signatures allow conspecifics to discern territorial boundaries, reproductive readiness, and individual identity purely through olfactory inspection.
On This Page
- Unraveling the Biochemical Architecture of Feline Chemical Signatures
- Olfactory Processing and Sensory Reception Mechanisms
- Ecological Functions of Scent Marking in Feline Populations
- Methodological Advances in Chemical Ecology and Biomarker Discovery
- Comparative Mammalian Scent Signaling and Evolutionary Parallels
Unraveling the Biochemical Architecture of Feline Chemical Signatures
The investigation into feline urine composition requires advanced analytical chemistry techniques to decode the intricate mixture of proteins, lipids, and small organic molecules. Researchers employ high-performance liquid chromatography and mass spectrometry to isolate specific compounds responsible for transmitting unique individual identity markers. Understanding these molecular structures helps scientists map out the physiological pathways that produce such durable and informative olfactory signals within domestic felines.
Molecular Composition and Volatile Organic Compounds
The identification signal resides within a complex matrix of aqueous urea, creatinine, and specialized carrier proteins known as felins. These urinary proteins bind specific volatile organic compounds, regulating their release rate into the surrounding air over extended periods. Without this specialized protein binding mechanism, the volatile markers would evaporate too quickly to serve as effective long-term territorial beacons for passing cats. Analytical evaluations demonstrate that the exact ratio of these carrier proteins varies distinctly among individuals, creating a unique biochemical fingerprint. This variation ensures that no two feline urine samples emit an identical olfactory profile, supporting individual recognition among populations.
Further chemical fractionation reveals that small sulfur-containing molecules contribute significantly to the sharp, characteristic odor associated with feline scent marking. These compounds undergo slow enzymatic degradation post-excretion, altering the signal's intensity and complexity as time progresses in the field. Consequently, reading animals can ascertain not only who left the mark but also the relative freshness and chronological age of the deposition. This temporal degradation acts as a natural clock, guiding foraging and patrol decisions for territorial cats navigating overlapping home ranges. Mathematical modeling of volatile diffusion rates helps researchers quantify how environmental temperature and humidity influence this chemical decay process.
To quantify the diffusion rate of volatile markers, we apply Fick's second law of diffusion adjusted for environmental boundary conditions. Let ##[C(x, t)]## represent the concentration of the volatile compound at distance ##[x]## and time ##[t]##:
In this governing differential equation, ##[D]## denotes the molecular diffusion coefficient of the urinary volatile compound in air. The parameter ##[k]## represents the first-order degradation constant driven by ambient atmospheric oxidation and microbial action. Solving this partial differential equation yields the spatial distribution profile utilized by investigating felines during olfactory searches.
We can also model the probability ##[P]## that a passing cat successfully detects the signal threshold ##[C_{th}]## over distance. Integrating the concentration function across a radial hemisphere gives the effective active space ##[V_{active}]## of the mark. This active space shrinks logarithmically as the degradation factor ##[k t]## increases throughout successive diurnal cycles. Field observations confirm that territorial patrolling behaviors adjust dynamically in response to these changing active space dimensions.
Genomic Regulation and Individual Specificity
The synthesis of these unique identification markers is governed by complex genetic loci that regulate major urinary proteins. Genetic polymorphism within these specific gene clusters ensures high variability across the broader feline population, preventing accidental signaling overlaps. Epigenetic factors and individual metabolic rates further fine-tune the final biochemical output, making each cat's chemical signature virtually unique. This biological mechanism resembles mammalian major histocompatibility complex scent signaling observed in various other vertebrate species. Researchers continue to sequence these genetic pathways to understand how selective pressures maintain such precise chemical diversity.
Investigating the metabolic pathways reveals that hepatic processing of amino acids directly influences the precursor molecules found in renal excretions. Dietary inputs can modulate these precursors, yet the core identification signal remains resilient against short-term nutritional fluctuations. This stability ensures that transient food availability does not compromise an individual's permanent social passport within its territory. Endocrinology studies further demonstrate that circulating androgen and estrogen levels upregulate specific protein expressions. Consequently, intact males and females produce distinct marker intensities compared to neutered counterparts.
To evaluate the genetic variance ##[\sigma^2_g]## across populations, we utilize the standard quantitative genetics estimator for phenotypic expression. Let ##[Y_{ij}]## represent the measured protein concentration for individual ##[i]## under condition ##[j]##:
Here, ##[\mu]## is the population mean, ##[G_i]## represents the random genetic effect of the ##[i]##-th feline, and ##[E_{ij}]## denotes environmental error. The heritability coefficient ##[H^2]## is calculated via the variance components:
Empirical calculations from recent biomarker studies indicate an exceptionally high heritability value ##[H^2 > 0.85]## for urinary protein profiles. This strong genetic grounding confirms that the identification signal operates as a reliable proxy for genetic relatedness and individual identity.
We can also model the mutation accumulation rate in these marker genes using a Poisson distribution framework. The probability of observing ##[k]## mutations across a genomic segment of length ##[L]## over evolutionary time ##[T]## is expressed as:
Where ##[\lambda]## represents the baseline per-nucleotide substitution rate. Maintaining high polymorphism in these loci is evolutionarily advantageous for avoiding inbreeding and managing territorial disputes efficiently. Mathematical simulations demonstrate that frequency-dependent selection actively preserves this chemical diversity within wild felid populations.
We Also Published
Olfactory Processing and Sensory Reception Mechanisms
Detecting and interpreting these sophisticated chemical markers requires highly specialized anatomical structures within the feline olfactory system. Felines possess both a main olfactory epithelium and a vomeronasal organ, commonly known as Jacobson's organ, located in the hard palate. When a cat investigates a urine deposition, it often performs the flehmen response, curling its upper lip to draw airborne molecules toward the vomeronasal ducts. This dual-processing capability allows the animal to separate general environmental odors from critical social identification signals encoded within the fluid matrix.
Neuroanatomy of the Vomeronasal Pathway
The vomeronasal organ houses specialized sensory receptor neurons that project directly to the accessory olfactory bulb within the central nervous system. Unlike the main olfactory system, which processes volatile general scents, the accessory pathway is tuned to non-volatile and semi-volatile high-molecular-weight proteins. This neural segregation ensures that the identification signature bypasses standard sensory filtering, gaining direct access to limbic processing centers. Consequently, encountering a familiar or unfamiliar urine mark instantly triggers strong behavioral, emotional, and physiological responses without conscious hesitation.
Histological examinations reveal a dense array of microvillar receptor cells expressing specific vomeronasal receptor gene families within the sensory epithelium. These receptors undergo rapid desensitization and resensitization cycles, enabling cats to process multiple distinct chemical exposures during intense territorial inspection patrols. Signal transduction within these receptor cells relies on specialized G-protein coupled cascades involving phospholipase C activation. This biochemical pathway amplifies weak chemical inputs into robust electrical action potentials traveling along the sensory nerve tracts.
To quantify the neural firing rate ##[R]## in response to varying ligand concentrations ##[L]##, neurophysiologists apply the Hill-Langmuir equation. Let ##[K_d]## be the dissociation constant of the receptor-ligand complex:
In this expression, ##[R_{max}]## represents the maximum achievable neural response rate, and ##[n]## is the Hill coefficient denoting cooperative binding. Experimental electrophysiological recordings yield Hill coefficients greater than ##[1.5]##, confirming cooperative interaction among receptor sites.
We can model the temporal adaptation of these sensory neurons using an exponential decay function for spike frequency over sustained exposure time ##[t]##:
Where ##[R_0]## is the initial peak firing rate, ##[\alpha]## is the neural adaptation rate constant, and ##[R_{steady}]## is the baseline tonic firing level. This rapid adaptation prevents sensory overload, allowing cats to detect sudden changes in marker composition as they investigate complex boundary sites.
Behavioral Responses to Identity Markers
Once the identification signal is successfully processed by the limbic system, the receiving cat exhibits distinct behavioral patterns depending on the marker's origin. If the urine deposition belongs to a familiar social group member, the inspecting cat typically displays calm, habituated behaviors or deposits an over-marking scent to reinforce communal bonds. Conversely, encountering the signal of an unknown interloper initiates defensive posturing, heightened vigilance, or deliberate avoidance strategies to prevent physical conflict. These behavioral switches demonstrate that the biological "ID card" effectively mediates social organization without requiring direct visual encounters.
Field studies record that dominant individuals invest more time investigating foreign marks compared to subordinates, reflecting differing territorial responsibilities within the colony structure. Furthermore, reproductive status heavily dictates reaction intensity, with intact adult males showing aggressive over-marking when detecting rival male signatures during peak breeding seasons. Understanding these behavioral algorithms provides profound insights into domestic cat welfare, space management, and multi-cat household dynamics. Behavioral veterinarians now utilize these chemical communication principles to resolve stress-related house-soiling and inter-cat aggression issues.
To analyze the probability of aggressive escalation ##[P_{agg}]## upon encountering a foreign ID signal, we construct a logistic regression model. Let ##[X_1]## be the intruder familiarity index and ##[X_2]## be the defender's hormonal status:
The coefficients ##[\beta_1]## and ##[\beta_2]## are estimated via maximum likelihood estimation from observational tracking data. Model validation confirms high predictive accuracy for forecasting territorial clashes in free-ranging feline populations.
We can also evaluate the expected time delay ##[T_{response}]## before a resident cat investigates a fresh mark using a hazard function framework. The hazard rate ##[h(t)]## of investigation is proportional to the initial signal concentration gradient:
Where ##[h_0]## is the baseline hazard and ##[\gamma]## is the sensitivity parameter. Shorter time delays correlate strongly with high-value core territory boundaries where intrusion costs are severe.
Ecological Functions of Scent Marking in Feline Populations
Scent marking serves as the cornerstone of feline spatial ecology, establishing invisible fences that regulate population density and resource allocation. By depositing urine ID cards at prominent environmental landmarks—such as tree trunks, fence posts, and rock outcrops—cats communicate their presence across time. This asynchronous communication prevents physical injury by allowing animals to partition their home ranges efficiently without engaging in direct combat. The stability of the urinary protein matrix ensures these territorial claims persist long after the depositor has moved to another sector.
Territorial Partitioning and Home Range Dynamics
Home ranges of domestic and wild felines often overlap significantly, yet core areas are fiercely defended through rigorous scent-marking routines. The identification signal embedded in the urine acts as a social deterrent, signaling residency status and competitive ability to potential trespassers. When an animal encounters a fresh marker, it assesses the relative strength and novelty of the chemical signature to gauge the resident's physical condition. If the signal indicates a robust, healthy adult, intruders frequently choose to detour around the contested zone, thereby avoiding costly physical confrontations.
Mathematical models of territorial boundary maintenance treat home range edges as equilibrium zones where opposing pressure vectors balance out. Let ##[F_{res}(x)]## be the residency pressure exerted by the owner at distance ##[x]## from the core:
And let ##[F_{int}(x)]## represent the intrusion pressure exerted by a neighboring rival approaching from the outside:
Where ##[D]## is the total distance between the two core activity centers. The stable territorial boundary ##[x^*]## occurs precisely where the two opposing pressure vectors reach dynamic equilibrium:
Solving for ##[x^*]## gives the precise spatial location of the scent-marked boundary line observed in field studies.
We can further analyze the energy expenditure ##[E_{mark}]## required to maintain a given perimeter length ##[L_{perim}]##. Assuming a constant deposition cost ##[c_m]## per unit length, the total daily energetic cost is modeled as:
Where ##[\nu]## is the renewal frequency required to prevent signal degradation below the detection threshold. Optimal foraging theory predicts that cats balance this marking cost against the caloric value of the defended resource patch.
Reproductive Signaling and Mate Selection
Beyond territorial defense, urine identification signals play a pivotal role during the breeding season by advertising reproductive availability and individual genetic quality. Intates release modified chemical profiles that broadcast ovulation status in females and competitive stamina in males. Prospective mates intercept these chemical bulletins along established travel corridors, using the embedded ID data to assess compatibility before initiating direct courtship. This pre-screening mechanism reduces the energetic costs associated with searching for receptive partners across fragmented habitats.
Biochemical analyses indicate that hormone-dependent metabolites alter the vapor pressure of urinary volatiles during peak fertility windows, creating an unmistakable olfactory beacon. Males detecting these heightened signals exhibit flehmen responses followed by intensive trailing behaviors designed to locate the signaling female. The precision of the ID signal ensures that males do not waste reproductive effort on non-receptive individuals or incompatible conspecifics. Evolutionary biologists view this system as an efficient filter that maximizes reproductive success while minimizing predation risks during mating excursions.
To quantify mate choice selectivity based on urinary peptide profiles, we apply Shannon's information theory index ##[H_{info}]## to the volatile bouquet:
Where ##[p_i]## represents the proportional abundance of the ##[i]##-th volatile compound in the total urinary emission. Higher information entropy ##[H_{info}]## correlates with complex genetic heterozygosity, which advertising felines project as an indicator of superior immune fitness.
We can model the probability of successful mate location ##[P_{mate}]## as a function of signal age ##[t]## and emitter density ##[\rho]##:
Where ##[R_{detect}]## is the maximum detection radius and ##[\delta]## is the chemical degradation rate. This equation highlights how rapid signal degradation maintains the temporal relevance of reproductive advertisements.
Methodological Advances in Chemical Ecology and Biomarker Discovery
Recent breakthroughs in analytical instrumentation have empowered researchers to isolate and characterize subtle biological signals that previously evaded detection. Traditional behavioral observations are now routinely combined with gas chromatography-mass spectrometry and metaproteomic sequencing to map complete chemical profiles. These multidisciplinary approaches allow scientists to dissect the exact molecular architecture of feline urine markers with unprecedented precision. Consequently, the discovery of the identification-like signal marks a major milestone in mammalian chemical ecology research.
Advanced Analytical Techniques in Biomarker Extraction
Isolating unstable volatile compounds from complex biological fluids requires specialized solid-phase microextraction fibers that capture trace organic molecules without altering their chemical structure. Researchers suspend these fibers in the headspace above urine samples to absorb airborne volatiles released by protein-ligand complexes. Subsequent thermal desorption directly into gas chromatographs separates individual chemical constituents for high-resolution mass spectral identification. This non-destructive sampling method preserves precious biological samples while yielding highly reproducible chromatographic fingerprints across multiple test subjects.
Metaproteomic profiling further complements these chromatographic methods by identifying the complete complement of urinary proteins secreted under varying physiological conditions. Researchers use liquid chromatography tandem mass spectrometry to sequence peptide fragments, matching them against established mammalian genomic databases. This pipeline has successfully cataloged dozens of novel carrier proteins and enzymatic degradation products specific to feline renal excretion. Such comprehensive datasets provide the foundational knowledge required to decode how cats synthesize and utilize their biological ID cards in natural environments.
To calculate the chromatographic resolution ##[R_s]## between two adjacent volatile peaks, analytical chemists apply the standard column efficiency formula:
In this equation, ##[t_{r1}]## and ##[t_{r2}]## represent the retention times of adjacent peaks, while ##[W_1]## and ##[W_2]## denote their respective baseline peak widths. Achieving a resolution value ##[R_s > 1.5]## ensures complete baseline separation of complex urinary volatile mixtures.
We can also evaluate column plate number ##[N]## to assess chromatographic efficiency using the retention time and peak width parameters:
High plate numbers exceeding ##[10^5]## theoretical plates are essential for resolving the minute structural differences between closely related feline urinary pheromones and carrier proteins.
Future Directions in Mammalian Pheromone Research
The identification of a robust biological ID signal in cat urine opens exciting avenues for future research across veterinary science, ethology, and conservation biology. Investigators aim to synthesize analogue compounds that can replicate these natural signaling properties for managing stress and behavioral issues in captive or domestic felines. Furthermore, expanding these analytical frameworks to wild felid species could revolutionize non-invasive population monitoring and endangered species conservation efforts globally. As analytical technologies continue to evolve, our understanding of the hidden chemical language governing mammalian societies will undoubtedly deepen.
Collaborative research initiatives are currently mapping the genetic conservation of these urinary signaling pathways across the entire Felidae family tree, from domestic cats to apex predators like tigers and leopards. Preliminary comparative data suggest that while the core protein structures remain conserved, lineage-specific volatile ligands provide species-specific isolation barriers. This broader evolutionary perspective helps scientists reconstruct the ancestral origins of chemical communication within mammalian lineages. Funding agencies are increasingly prioritizing these interdisciplinary studies due to their high translational value for animal welfare and wildlife management.
To estimate the sampling effort required to detect rare volatile variants across diverse wild populations, ecologists employ species accumulation curve modeling. Let ##[S(N)]## represent the number of distinct chemical variants discovered as a function of sample size ##[N]##:
Where ##[S_{max}]## is the estimated asymptotic total of chemical variants and ##[b]## is the scaling parameter governing discovery rate. Nonlinear regression fits confirm that extensive regional sampling is necessary to capture the full spectrum of intraspecific chemical diversity.
We can also project the cost-benefit ratio ##[CB]## of deploying synthetic analogue diffusers in multi-cat shelters using a linear programming optimization function:
Maximizing this ratio ensures that veterinary interventions utilizing synthetic ID signals achieve maximum stress-reduction efficacy while remaining economically viable for shelter operations.
Comparative Mammalian Scent Signaling and Evolutionary Parallels
The reliance on urinary chemical markers for individual identification is not unique to felines, representing a deeply conserved evolutionary strategy observed across diverse mammalian orders. Rodents, ungulates, and canids all utilize specialized protein-ligand complexes in their excretions to broadcast social status, territory ownership, and genetic compatibility. Comparing these parallel evolutionary adaptations provides crucial context for understanding how the feline ID signal fits into the broader tapestry of mammalian chemical ecology. Despite anatomical variations in olfactory apparatuses, the underlying biochemical logic remains remarkably consistent across species.
Cross-Species Analysis of Urinary Protein Carriers
Mammalian urinary proteins frequently belong to the lipocalin superfamily, characterized by a conserved barrel-like structure that encapsulates hydrophobic volatile molecules securely. In mice, these are known as major urinary proteins, whereas rats utilize similar alpha-2-uromobulins and felines rely on cauxin and felin variants. This convergence of protein architecture highlights strong selective pressures favoring stable carriers that can withstand harsh environmental exposure. Analyzing the amino acid sequences of these carrier proteins reveals ancient gene duplication events that predated the divergence of modern mammalian lineages.
The functional convergence extends to the ways recipient animals process these biochemical messages using vomeronasal and main olfactory pathways. Across rodents and carnivores, accessory olfactory bulb activation triggers stereotyped neuroendocrine responses that modulate aggression, parental care, and sexual maturation. This shared neural circuitry underscores the profound evolutionary importance of chemical communication in maintaining social cohesion and reproductive success. Researchers continue to explore these comparative models to uncover universal principles governing mammalian olfactory processing and signal evolution.
To quantify the evolutionary divergence between mammalian carrier protein sequences, bioinformaticians calculate the evolutionary distance ##[d_{XY}]## using Jukes-Cantor corrected substitution models. Let ##[p]## be the proportion of differing amino acid sites between two species:
Applying this formula to feline cauxin versus murine major urinary proteins reveals deep phylogenetic divergence times exceeding tens of millions of years.
We can also model the rate of protein evolution using the ratio of non-synonymous to synonymous substitution rates ##[\omega = d_N / d_S]##:
Empirical estimates yielding ##[\omega > 1]## across specific ligand-binding pockets confirm positive Darwinian selection actively diversifying these recognition sites to maximize individual distinctiveness.
Implications for Synthetic Biology and Artificial Olfaction
Decoding the chemical architecture of feline identification signals provides inspiration for developing advanced artificial olfaction systems and electronic noses. Engineers seek to replicate the selective binding properties of mammalian lipocalins in synthetic polymer matrices to detect specific biomarkers in environmental or medical diagnostics. By mimicking the slow-release mechanisms of urinary proteins, technological applications can achieve durable, long-lasting scent deployment for pest control or wildlife management. These cross-disciplinary innovations demonstrate how fundamental biological discoveries translate into practical engineering solutions.
Furthermore, understanding how felines process complex olfactory mixtures aids in designing better behavioral enrichment protocols for captive animals in zoos and sanctuaries. Recreating natural chemical landscapes helps alleviate chronic stress and encourages species-typical exploration behaviors that improve overall animal welfare standards. As researchers continue to publish detailed analyses of biological ID signals, the synergy between chemical ecology and applied technology will undoubtedly accelerate. This ongoing scientific journey underscores the profound complexity hidden within everyday biological phenomena.
To model the sensitivity threshold ##[S_{sensor}]## of an artificial lipocalin-based sensor array, engineers apply the Langmuir adsorption isotherm for surface binding:
Where ##[\theta]## represents the fraction of surface binding sites occupied by target volatile molecules, and ##[K_a]## is the adsorption equilibrium constant. Optimizing ##[K_a]## ensures high sensitivity for detecting trace urinary markers in complex background atmospheres.
We can also evaluate the signal-to-noise ratio ##[SNR]## of the artificial sensor output using variance metrics:
Maximizing this ratio through advanced neural network filtering enables electronic noses to reliably identify individual feline signatures even in highly contaminated environmental settings.
From our network :
- EV 2.0: The Solid-State Battery Breakthrough and Global Factory ExpansionDiscover the impact of the Solid-State Battery Breakthrough on the EV market. Learn about CATL and BYD stock growth, global factory expansion in Europe, and the future of EV 2.0 technology.
- Mastering DB2 12.1 Instance Design: A Technical Deep Dive into Modern Database ArchitectureComprehensive guide to DB2 12.1 Instance Design. Explore architectural components, HADR setup, buffer pool tuning, and security policies for IBM DB2 12.1. Includes 10 functional SQL and Shell samples.
- 10 Physics Numerical Problems with Solutions for IIT JEEPrepare for IIT JEE with 10 physics numerical problems, complete with detailed solutions and conceptual explanations. Ideal for mastering kinematics, thermodynamics, electromagnetism, and optics.
- Analyzing Trump Deportation Numbers Insights Into The 2026 Immigration Crackdown
- AI-Powered 'Precision Diagnostic' Replaces Standard GRE Score ReportsDiscover the new GRE Precision Diagnostic. Learn how AI-powered behavioral analytics and time-to-solve tracking are replacing standard GRE score reports to empower students.
- Trump Political Strategy How Geopolitical Stunts Serve As Media Diversions
- 98% of Global MBA Programs Now Prefer GRE Over GMAT Focus EditionExplore why 98% of global MBA programs now prefer the GRE over GMAT Focus. Learn about the shorter GRE format, verbal logic importance, and strategic versatility for students.
- Vite 6/7 'Cold Start' Regression in Massive Module GraphsIn-depth analysis of Vite 6/7 cold start regressions in massive module graphs. Learn about barrel file issues, pre-bundling optimizations, and how to improve Vite dev server performance.
- Mastering DB2 LUW v12 Tables: A Comprehensive Technical GuideComprehensive guide on DB2 LUW v12 tables. Explore CREATE TABLE syntax, BLU Acceleration, range partitioning, data types, and security features for IBM DB2 LUW v12.
RESOURCES
- Signatures of branched-chain fatty acids derived from a kidney ...cell.comAug 19, 2026 ... ∙ Koziel, J.A. ∙ Li, J.Z.. Simultaneous chemical and sensory analysis of domestic cat urine and feces with headspace solid-phase ...
- A comparative profile of urinary scent signals of two endangered ...frontiersin.orgJun 27, 2023 ... ... chemical ecology of endangered species. Because both subspecies are officially classified as the mainland leopard cat (Prionailurus ...
- Signatures of branched-chain fatty acids derived from a kidney ...sciencedirect.comUsing behavior-guided chemistry, we identify a structurally unusual repertoire of urinary BFAs whose compositional profiles are individually distinctive, stable ...
- Sprayed Urine Emits a Pungent Odor due to its Increased Adhesion ...pubmed.ncbi.nlm.nih.govApr 10, 2024 ... The sprayed urine is recognized as a chemical signal for territorial ownership of their habitats. ... urine for chemical communication…
- Common scents? A review of potentially shared chemical signals in ...pmc.ncbi.nlm.nih.govThe process may start with the analysis of urine as the general source of the chemical signal. ... cat and wolf urine (Berton et…
- Identification of volatile components of bobcat (Lynx rufus) urinelink.springer.comJournal of Chemical Ecology; Article. Identification of volatile components of ... Chemical Signals: Vertebrates and Aquatic Invertebrates. Plenum, New ...
- The Chemical Ecology of Elephants: 21st Century Additions to Our ...mdpi.comSep 30, 2021 ... Chemical analysis of preovulatory female African elephant urine: A search for putative pheromones. In Chemical Signals in Vertebrates 10 ...
- Chemical profiles of volatile compounds emitted from cat bodies. a...researchgate.netOther sources of chemical signals (e.g., urine, feces, and anal gland secretions) in cats have been identified and their potential functions have been ...
- How pheromones signal mating cues in tilapia | ScienceDailysciencedaily.comSep 1, 2014 ... Scientists have now identified such a signal molecule in the urine ... Max Planck Institute for Chemical Ecology. "Ready for…
- Pheromones of Tiger and Other Big Cats - NCBIncbi.nlm.nih.govChemical analysis of the urine of a tiger cub revealed traces of free fatty ... Evolution of chemical signals in the Asian elephant, Elephas…
- Researchers identify a pheromone in the urine of male tilapia fish ...phys.orgAug 29, 2014 ... The exchange of chemical signals between organisms is considered the oldest form of communication. Acting as messenger molecules, ...
- Single compounds elicit complex behavioural responses in wild ...nature.comAug 22, 2018 ... ... cat urine at ca. 5 ng L−1 or above. Moreover, some studies have ... in Chemical Signals in Vertebrates…
- Reverse chemical ecology: Olfactory proteins from the giant panda ...pnas.orgAnimal behavior studies and chemical analysis of specific secretions have indicated urine and the perianal gland secretions as the biological fluids responsible ...
- Take a good catch at the scat: carboxylic and sulfonic acid profiles ...tandfonline.comSource: Journal of Chemical Ecology. Three mammal species distinction through ... GC × GC-MS-Based Volatile Profiling of Male Domestic Cat Urine and the ...
- Investigating a Systematic and Widespread Misidentification in the ...pubs.acs.orgOct 24, 2025 ... PAGln and PAGly are urinary metabolites of microbial-hepatic phenylalanine metabolism, with the former linked to chemical signaling and ...
0 Comments